P47250
Gene name |
gyrA |
Protein name |
DNA gyrase subunit A |
Names |
|
Species |
Mycoplasma genitalium (strain ATCC 33530 / DSM 19775 / NCTC 10195 / G37) (Mycoplasmoides genitalium) |
KEGG Pathway |
mge:MG_004 |
EC number |
5.6.2.2: Enzymes altering nucleic acid conformation |
Protein Class |
|
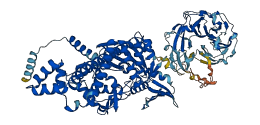
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for P47250
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-P47250-F1 | Predicted | AlphaFoldDB |
No variants for P47250
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for P47250 | |||||
No associated diseases with P47250
7 regional properties for P47250
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | DNA topoisomerase, type IIA, domain A | 23 - 485 | IPR002205 |
| repeat | DNA gyrase/topoisomerase IV, subunit A, C-terminal repeat | 517 - 562 | IPR006691-1 |
| repeat | DNA gyrase/topoisomerase IV, subunit A, C-terminal repeat | 566 - 615 | IPR006691-2 |
| repeat | DNA gyrase/topoisomerase IV, subunit A, C-terminal repeat | 621 - 661 | IPR006691-3 |
| repeat | DNA gyrase/topoisomerase IV, subunit A, C-terminal repeat | 668 - 711 | IPR006691-4 |
| repeat | DNA gyrase/topoisomerase IV, subunit A, C-terminal repeat | 720 - 760 | IPR006691-5 |
| repeat | DNA gyrase/topoisomerase IV, subunit A, C-terminal repeat | 769 - 812 | IPR006691-6 |
Functions
| Description | ||
|---|---|---|
| EC Number | 5.6.2.2 | Enzymes altering nucleic acid conformation |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
3 GO annotations of cellular component
| Name | Definition |
|---|---|
| chromosome | A structure composed of a very long molecule of DNA and associated proteins (e.g. histones) that carries hereditary information. |
| cytoplasm | The contents of a cell excluding the plasma membrane and nucleus, but including other subcellular structures. |
| DNA topoisomerase type II (double strand cut, ATP-hydrolyzing) complex | Complex that possesses DNA topoisomerase II (double strand cut, ATP-hydrolyzing) activity. |
3 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| DNA binding | Any molecular function by which a gene product interacts selectively and non-covalently with DNA (deoxyribonucleic acid). |
| DNA negative supercoiling activity | Catalytic introduction of negative supercoils into a DNA molecule or region thereof. In bacteria, negative supercoils are only introduced by DNA gyrase, a type II topoisomerase, but not all DNA gyrases are capable of introducing supercoils. In bacteria, the level of supercoiling varies widely between species and has been characterized properly in only a handful of organisms. The best characterized enzyme, from E.coli, is exceptionally proficient at supercoiling and this ability is not representative of all bacteria. |
2 GO annotations of biological process
| Name | Definition |
|---|---|
| DNA topological change | The process in which a transformation is induced in the topological structure of a double-stranded DNA helix, resulting in a change in linking number. |
| DNA-templated DNA replication | A DNA replication process that uses parental DNA as a template for the DNA-dependent DNA polymerases that synthesize the new strands. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MAKQQDQVDK | IRENLDNSTV | KSISLANELE | RSFMEYAMSV | IVARALPDAR | DGLKPVHRRV |
| 70 | 80 | 90 | 100 | 110 | 120 |
| LYGAYIGGMH | HDRPFKKSAR | IVGDVMSKFH | PHGDMAIYDT | MSRMAQDFSL | RYLLIDGHGN |
| 130 | 140 | 150 | 160 | 170 | 180 |
| FGSIDGDRPA | AQRYTEARLS | KLAAELLKDI | DKDTVDFIAN | YDGEEKEPTV | LPAAFPNLLA |
| 190 | 200 | 210 | 220 | 230 | 240 |
| NGSSGIAVGM | STSIPSHNLS | ELIAGLIMLI | DNPQCTFQEL | LTVIKGPDFP | TGANIIYTKG |
| 250 | 260 | 270 | 280 | 290 | 300 |
| IESYFETGKG | NVVIRSKVEI | EQLQTRSALV | VTEIPYMVNK | TTLIEKIVEL | VKAEEISGIA |
| 310 | 320 | 330 | 340 | 350 | 360 |
| DIRDESSREG | IRLVIEVKRD | TVPEVLLNQL | FKSTRLQVRF | PVNMLALVKG | APVLLNMKQA |
| 370 | 380 | 390 | 400 | 410 | 420 |
| LEVYLDHQID | VLVRKTKFVL | NKQQERYHIL | SGLLIAALNI | DEVVAIIKKS | ANNQEAINTL |
| 430 | 440 | 450 | 460 | 470 | 480 |
| NTKFKLDEIQ | AKAVLDMRLR | SLSVLEVNKL | QTEQKELKDS | IEFCKKVLAD | QKLQLKIIKE |
| 490 | 500 | 510 | 520 | 530 | 540 |
| ELQKINDQFG | DERRSEILYD | ISEEIDDESL | IKVENVVITM | STNGYLKRIG | VDAYNLQHRG |
| 550 | 560 | 570 | 580 | 590 | 600 |
| GVGVKGLTTY | VDDSISQLLV | CSTHSDLLFF | TDKGKVYRIR | AHQIPYGFRT | NKGIPAVNLI |
| 610 | 620 | 630 | 640 | 650 | 660 |
| KIEKDERICS | LLSVNNYDDG | YFFFCTKNGI | VKRTSLNEFI | NILSNGKRAI | SFDDNDTLYS |
| 670 | 680 | 690 | 700 | 710 | 720 |
| VIKTHGNDEI | FIGSTNGFVV | RFHENQLRVL | SRTARGVFGI | SLNKGEFVNG | LSTSSNGSLL |
| 730 | 740 | 750 | 760 | 770 | 780 |
| LSVGQNGIGK | LTSIDKYRLT | KRNAKGVKTL | RVTDRTGPVV | TTTTVFGNED | LLMISSAGKI |
| 790 | 800 | 810 | 820 | 830 | |
| VRTSLQELSE | QGKNTSGVKL | IRLKDNERLE | RVTIFKEELE | DKEMQLEDVG | SKQITQ |