P47027
Gene name |
DPB11 (YJL090C, J0918) |
Protein name |
DNA replication regulator DPB11 |
Names |
|
Species |
Saccharomyces cerevisiae (strain ATCC 204508 / S288c) (Baker's yeast) |
KEGG Pathway |
sce:YJL090C |
EC number |
|
Protein Class |
|
Descriptions
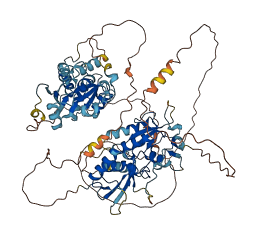
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for P47027
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-P47027-F1 | Predicted | AlphaFoldDB |
15 variants for P47027
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| s10-264833 | 72 | Q>K | No | SGRP | |
| s10-264628 | 140 | S>N | No | SGRP | |
| s10-264162 | 295 | Q>H | No | SGRP | |
| s10-264160 | 296 | Q>R | No | SGRP | |
| s10-264149 | 300 | T>A | No | SGRP | |
| s10-264098 | 317 | E>K | No | SGRP | |
| s10-263877 | 390 | D>E | No | SGRP | |
| s10-263503 | 515 | C>Y | No | SGRP | |
| s10-263476 | 524 | G>D | No | SGRP | |
| s10-263460 | 529 | K>N | No | SGRP | |
| s10-263239 | 603 | Y>C | No | SGRP | |
| s10-263080 | 656 | R>K | No | SGRP | |
| s10-262979 | 690 | V>F | No | SGRP | |
| s10-262813 | 745 | A>V | No | SGRP | |
| s10-262778 | 757 | N>Y | No | SGRP |
No associated diseases with P47027
6 regional properties for P47027
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | Coagulation factor 5/8 C-terminal domain | 276 - 427 | IPR000421-1 |
| domain | Coagulation factor 5/8 C-terminal domain | 433 - 592 | IPR000421-2 |
| domain | CUB domain | 28 - 142 | IPR000859-1 |
| domain | CUB domain | 149 - 267 | IPR000859-2 |
| domain | MAM domain | 641 - 802 | IPR000998 |
| domain | Neuropilin, C-terminal | 853 - 931 | IPR022579 |
3 GO annotations of cellular component
| Name | Definition |
|---|---|
| DNA replication preinitiation complex | A protein-DNA complex assembled at eukaryotic DNA replication origins immediately prior to the initiation of DNA replication. The preinitiation complex is formed by the assembly of additional proteins onto an existing prereplicative complex. In budding yeast, the additional proteins might include Cdc45p, Sld2p, Sld3p, Dpb11p, DNA polymerases, and others; in fission yeast the GINS complex is present. |
| nucleus | A membrane-bounded organelle of eukaryotic cells in which chromosomes are housed and replicated. In most cells, the nucleus contains all of the cell's chromosomes except the organellar chromosomes, and is the site of RNA synthesis and processing. In some species, or in specialized cell types, RNA metabolism or DNA replication may be absent. |
| replication fork | The Y-shaped region of a replicating DNA molecule, resulting from the separation of the DNA strands and in which the synthesis of new strands takes place. Also includes associated protein complexes. |
2 GO annotations of molecular function
| Name | Definition |
|---|---|
| DNA polymerase binding | Binding to a DNA polymerase. |
| protein kinase activator activity | Binds to and increases the activity of a protein kinase, an enzyme which phosphorylates a protein. |
10 GO annotations of biological process
| Name | Definition |
|---|---|
| DNA replication checkpoint signaling | A signal transduction process that contributes to a DNA replication checkpoint, that prevents the initiation of nuclear division until DNA replication is complete, thereby ensuring that progeny inherit a full complement of the genome. |
| DNA replication initiation | The process in which DNA-dependent DNA replication is started; this begins with the ATP dependent loading of an initiator complex onto the DNA, this is followed by DNA melting and helicase activity. In bacteria, the gene products that enable the helicase activity are loaded after the initial melting and in archaea and eukaryotes, the gene products that enable the helicase activity are inactive when they are loaded and subsequently activate. |
| double-strand break repair via break-induced replication | The error-free repair of a double-strand break in DNA in which the centromere-proximal end of a broken chromosome searches for a homologous region in an intact chromosome. DNA synthesis initiates from the 3' end of the invading DNA strand, using the intact chromosome as the template, and progresses to the end of the chromosome. |
| mating type switching | The conversion of a single-cell organism from one mating type to another by the precise replacement of a DNA sequence at the expressed mating type locus with a copy of a sequence from a donor locus. |
| mitotic DNA replication checkpoint signaling | A signal transduction process that contributes to a mitotic DNA replication checkpoint. |
| mitotic G2 DNA damage checkpoint signaling | A mitotic cell cycle checkpoint that detects and negatively regulates progression through the G2/M transition of the cell cycle in response to DNA damage. |
| positive regulation of DNA replication origin binding | Any process that activates or increases the frequency, rate or extent of DNA replication origin binding. |
| positive regulation of protein phosphorylation | Any process that activates or increases the frequency, rate or extent of addition of phosphate groups to amino acids within a protein. |
| recombinational repair | A DNA repair process that involves the exchange, reciprocal or nonreciprocal, of genetic material between the broken DNA molecule and a homologous DNA region. |
| regulation of mitotic DNA replication initiation | Any process that modulates the frequency, rate or extent of DNA replication initiation involved in mitotic DNA replication. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MKPFQGITFC | PTAINNEILA | KKISKKIIKL | GGIFSKDLTR | QVNVLVVGST | TNTNKFKFAV |
| 70 | 80 | 90 | 100 | 110 | 120 |
| KHRFDIIFID | IQAIDDIYQL | WLSGENILPD | SNTATMTGST | YEMLKILYRR | FSFKYLHNFN |
| 130 | 140 | 150 | 160 | 170 | 180 |
| IFIGRITDTN | ITSIDSLVRS | IKKLGCSSYN | YQNFVIKDTS | SHNDDDDQGQ | NGQISIFVTD |
| 190 | 200 | 210 | 220 | 230 | 240 |
| TLLGARVNAA | IEQNIPIVHF | KWILDCQKRS | ALLPYDPYYL | LPNIKDLPYD | SIGSNSCDCW |
| 250 | 260 | 270 | 280 | 290 | 300 |
| DKINTTFPTN | IDAQSSLQRQ | QSSSTLTPSL | PKTSSLLNKF | KPKGEKIWDK | AMSLQQHSKT |
| 310 | 320 | 330 | 340 | 350 | 360 |
| NFSVLGQSPL | SINNKQEDLS | DNSTLIFKNC | AFIIHHIFPG | NHRSILTKIV | VQNGGKIETS |
| 370 | 380 | 390 | 400 | 410 | 420 |
| YLSGIYDHSY | YIIPSNKALD | SFNDLPEIID | DNDGIVTEFF | IERCLYYQKL | LHPIDLWSKP |
| 430 | 440 | 450 | 460 | 470 | 480 |
| FLSTIEFQVS | SSSKLLHHEF | SSSPFLNVTI | TGFSGVELLH | LTKVLNLLKP | MGINYVEYLN |
| 490 | 500 | 510 | 520 | 530 | 540 |
| KSTDILLINL | AALPSIPKTH | PLWSNEFSDL | FTQFCINNNN | DDPGDNNRKD | FQNNSILRNS |
| 550 | 560 | 570 | 580 | 590 | 600 |
| MKRKIEYIKK | FHSIPVVTPA | FIFKLLSAAS | GENNEIFLNN | IKWCIICPRG | HKDDFKCKIK |
| 610 | 620 | 630 | 640 | 650 | 660 |
| KPYYTSISSE | KKYQNNDPKI | DKTILLKRNN | SSLSEHSMKD | TKNELLQKIR | ETDSGRKKRS |
| 670 | 680 | 690 | 700 | 710 | 720 |
| VSSSIMDVSS | ERQMPDTKRI | KLESLPKNFV | PKQIKRTTSW | GTIMSENVPT | EQPTAISNPE |
| 730 | 740 | 750 | 760 | ||
| EIPRTEEVSH | TQVTYGSIQD | KKRTASLEKP | MRRQTRNQTK | ELDS |