P38838
Gene name |
WSS1 (YHR134W) |
Protein name |
DNA-dependent metalloprotease WSS1 |
Names |
DNA damage response protein WSS1, SUMO-dependent isopeptidase WSS1, Weak suppressor of SMT3 protein 1 |
Species |
Saccharomyces cerevisiae (strain ATCC 204508 / S288c) (Baker's yeast) |
KEGG Pathway |
sce:YHR134W |
EC number |
|
Protein Class |
|
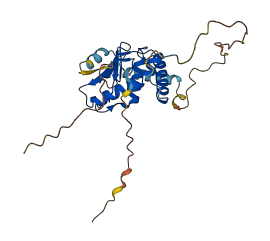
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for P38838
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-P38838-F1 | Predicted | AlphaFoldDB |
9 variants for P38838
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| s08-371758 | 3 | T>A | No | SGRP | |
| s08-371818 | 23 | P>A | No | SGRP | |
| s08-371836 | 29 | I>V | No | SGRP | |
| s08-372001 | 84 | V>I | No | SGRP | |
| s08-372175 | 142 | V>I | No | SGRP | |
| s08-372242 | 164 | N>S | No | SGRP | |
| s08-372393 | 214 | F>L | No | SGRP | |
| s08-372473 | 241 | I>N | No | SGRP | |
| s08-372536 | 262 | L>P | No | SGRP |
No associated diseases with P38838
1 regional properties for P38838
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | WLM domain | 20 - 221 | IPR013536 |
Functions
2 GO annotations of cellular component
| Name | Definition |
|---|---|
| fungal-type vacuole | A vacuole that has both lytic and storage functions. The fungal vacuole is a large, membrane-bounded organelle that functions as a reservoir for the storage of small molecules (including polyphosphate, amino acids, several divalent cations (e.g. calcium), other ions, and other small molecules) as well as being the primary compartment for degradation. It is an acidic compartment, containing an ensemble of acid hydrolases. At least in S. cerevisiae, there are indications that the morphology of the vacuole is variable and correlated with the cell cycle, with logarithmically growing cells having a multilobed, reticulated vacuole, while stationary phase cells contain a single large structure. |
| nuclear envelope | The double lipid bilayer enclosing the nucleus and separating its contents from the rest of the cytoplasm; includes the intermembrane space, a gap of width 20-40 nm (also called the perinuclear space). |
5 GO annotations of molecular function
| Name | Definition |
|---|---|
| metal ion binding | Binding to a metal ion. |
| metalloendopeptidase activity | Catalysis of the hydrolysis of internal, alpha-peptide bonds in a polypeptide chain by a mechanism in which water acts as a nucleophile, one or two metal ions hold the water molecule in place, and charged amino acid side chains are ligands for the metal ions. |
| metallopeptidase activity | Catalysis of the hydrolysis of peptide bonds by a mechanism in which water acts as a nucleophile, one or two metal ions hold the water molecule in place, and charged amino acid side chains are ligands for the metal ions. |
| SUMO binding | Binding to the small ubiquitin-like protein SUMO. |
| SUMO ligase activity | Catalysis of the transfer of SUMO to a substrate protein via the reaction X-SUMO + S --> X + S-SUMO, where X is either an E2 or E3 enzyme, the X-SUMO linkage is a thioester bond, and the S-SUMO linkage is an isopeptide bond between the C-terminal amino acid of SUMO and the epsilon-amino group of lysine residues in the substrate. |
10 GO annotations of biological process
| Name | Definition |
|---|---|
| cellular response to DNA damage stimulus | Any process that results in a change in state or activity of a cell (in terms of movement, secretion, enzyme production, gene expression, etc.) as a result of a stimulus indicating damage to its DNA from environmental insults or errors during metabolism. |
| histone catabolic process | The chemical reactions and pathways resulting in the breakdown of a histone protein by individual cells. |
| protein autosumoylation | The sumoylation by a protein of one or more of its own amino acid residues, or residues on an identical protein. |
| protein sumoylation | The process in which a SUMO protein (small ubiquitin-related modifier) is conjugated to a target protein via an isopeptide bond between the carboxy-terminus of SUMO with an epsilon-amino group of a lysine residue of the target protein. |
| protein-DNA covalent cross-linking repair | The removal of covalent cross-link between DNA and a protein. |
| proteolysis | The hydrolysis of proteins into smaller polypeptides and/or amino acids by cleavage of their peptide bonds. |
| replication-born double-strand break repair via sister chromatid exchange | The repair of a replication-born double-strand DNA break in which the DNA molecule is repaired using the homologous sequence of the sister chromatid which serves as a template to repair the breaks. |
| response to UV-B | Any process that results in a change in state or activity of a cell or an organism (in terms of movement, secretion, enzyme production, gene expression, etc.) as a result of a UV-B radiation stimulus. UV-B radiation (UV-B light) spans the wavelengths 280 to 315 nm. |
| response to UV-C | Any process that results in a change in state or activity of a cell or an organism (in terms of movement, secretion, enzyme production, gene expression, etc.) as a result of a UV-C radiation stimulus. UV-C radiation (UV-C light) spans the wavelengths 100 to 280 nm. |
| translesion synthesis | The replication of damaged DNA by synthesis across a lesion in the template strand; a specialized DNA polymerase or replication complex inserts a defined nucleotide across from the lesion which allows DNA synthesis to continue beyond the lesion. This process can be mutagenic depending on the damaged nucleotide and the inserted nucleotide. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MKTEGIKSPS | AKYHDMAGSQ | RIPHKNPHIQ | KVAVLQSKPN | KEDALNLIKE | IAHKVSYLMK |
| 70 | 80 | 90 | 100 | 110 | 120 |
| ENHFKVTNLV | EFYPRDQRLL | GMNVNHGSKI | MLRLRCSTDE | FQFLPMECIM | GTMLHELTHN |
| 130 | 140 | 150 | 160 | 170 | 180 |
| LFGPHDKKFY | NKLDELIGRQ | WVIEQRGLYD | TFLGNGQRLG | GRANLRSNRY | PMTGISTNTG |
| 190 | 200 | 210 | 220 | 230 | 240 |
| IVRKRGKGVK | LGSLHPEGIS | SIDRGNSPRE | LAAFAAERRY | RDDRWCGETK | NNKDQIISDN |
| 250 | 260 | ||||
| ISSSLEVVIL | DDDDEVLPGD | TLIEVIDLT |