P28876
Gene name |
pma2 (SPCC1020.01c, SPCC1393.01) |
Protein name |
Plasma membrane ATPase 2 |
Names |
Proton pump 2 |
Species |
Schizosaccharomyces pombe (strain 972 / ATCC 24843) (Fission yeast) |
KEGG Pathway |
spo:SPCC1020.01c |
EC number |
7.1.2.1: Hydron translocation linked to the hydrolysis of a nucleoside triphosphate |
Protein Class |
|
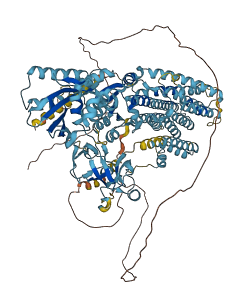
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for P28876
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-P28876-F1 | Predicted | AlphaFoldDB |
No variants for P28876
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for P28876 | |||||
No associated diseases with P28876
Functions
| Description | ||
|---|---|---|
| EC Number | 7.1.2.1 | Hydron translocation linked to the hydrolysis of a nucleoside triphosphate |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
4 GO annotations of cellular component
| Name | Definition |
|---|---|
| cell division site | The eventual plane of cell division (also known as cell cleavage or cytokinesis) in a dividing cell. In Eukaryotes, the cleavage apparatus, composed of septin structures and the actomyosin contractile ring, forms along this plane, and the mitotic, or meiotic, spindle is aligned perpendicular to the division plane. In bacteria, the cell division site is generally located at mid-cell and is the site at which the cytoskeletal structure, the Z-ring, assembles. |
| cell tip | The region at the end of the longest axis of a cylindrical or elongated cell. |
| integral component of membrane | The component of a membrane consisting of the gene products and protein complexes having at least some part of their peptide sequence embedded in the hydrophobic region of the membrane. |
| plasma membrane | The membrane surrounding a cell that separates the cell from its external environment. It consists of a phospholipid bilayer and associated proteins. |
5 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| ATP hydrolysis activity | Catalysis of the reaction: ATP + H2O = ADP + H+ phosphate. ATP hydrolysis is used in some reactions as an energy source, for example to catalyze a reaction or drive transport against a concentration gradient. |
| metal ion binding | Binding to a metal ion. |
| P-type ion transporter activity | Enables the transfer of a solute or solutes from one side of a membrane to the other according to the reaction: ATP + H2O = ADP + phosphate, to directly drive the transport of ions across a membrane. The reaction is characterized by the transient formation of a high-energy aspartyl-phosphoryl-enzyme intermediate. |
| P-type proton-exporting transporter activity | Enables the transfer of protons from one side of a membrane to the other according to the reaction: ATP + H2O + H+(in) -> ADP + phosphate + H+(out). These transporters use a phosphorylative mechanism, which have a phosphorylated intermediate state during the ion transport cycle. |
4 GO annotations of biological process
| Name | Definition |
|---|---|
| ion transmembrane transport | A process in which an ion is transported across a membrane. |
| proton export across plasma membrane | The directed movement of hydrogen ions (protons) from inside a cell, across the plasma membrane and into the extracellular region. |
| proton transmembrane transport | The directed movement of a proton across a membrane. |
| regulation of intracellular pH | Any process that modulates the internal pH of a cell, measured by the concentration of the hydrogen ion. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MQRNNGEGRP | EGMHRISRFL | HGNPFKNNAS | PQDDSTTRTE | VYEEGGVEDS | AVDYDNASGN |
| 70 | 80 | 90 | 100 | 110 | 120 |
| AAPRLTAAPN | THAQQANLQS | GNTSITHETQ | STSRGQEATT | SPSLSASHEK | PARPQTGEGS |
| 130 | 140 | 150 | 160 | 170 | 180 |
| DNEDEDEDID | ALIEDLYSQD | QEEEQVEEEE | SPGPAGAAKV | VPEELLETDP | KYGLTESEVE |
| 190 | 200 | 210 | 220 | 230 | 240 |
| ERKKKYGLNQ | MKEEKTNNIK | KFLSFFVGPI | QFVMELAAAL | AAGLRDWVDF | GVICALLLLN |
| 250 | 260 | 270 | 280 | 290 | 300 |
| ATVGFVQEYQ | AGSIVDELKK | TMALKASVLR | DGRVKEIEAS | EIVPGDILHL | DEGTICPADG |
| 310 | 320 | 330 | 340 | 350 | 360 |
| RLITKDCFLQ | VDQSAITGES | LAVDKHQNDT | MYSSSTVKRG | EAFMVVTATA | DSTFVGRAAS |
| 370 | 380 | 390 | 400 | 410 | 420 |
| LVGAAGQSQG | HFTEVLNGIG | TILLVLVILT | LLCIYTAAFY | RSVRLAALLE | YTLAITIIGV |
| 430 | 440 | 450 | 460 | 470 | 480 |
| PVGLPAVVTT | TMAVGAAYLA | KKKAIVQKLS | AIESLAGVEI | LCSDKTGTLT | KNRLSLGEPY |
| 490 | 500 | 510 | 520 | 530 | 540 |
| CVEGVSPDDL | MLTACLASSR | KKKGLDAIDK | AFLKALRNYP | KAKDQLSKYK | VLDFHPFDPV |
| 550 | 560 | 570 | 580 | 590 | 600 |
| SKKITAYVEA | PDGQRITCVK | GAPLWVFKTV | QDDHEVPEAI | TDAYREQVND | MASRGFRSLG |
| 610 | 620 | 630 | 640 | 650 | 660 |
| VARKADGKQW | EILGIMPCSD | PPRHDTARTI | HEAIGLGLRI | KMLTGDAVGI | AKETARQLGM |
| 670 | 680 | 690 | 700 | 710 | 720 |
| GTNVYNAERL | GLSGGGDMPG | SEVNDFVEAA | DGFAEVFPQH | KYAVVDILQQ | RGYLVAMTGD |
| 730 | 740 | 750 | 760 | 770 | 780 |
| GVNDAPSLKK | ADAGIAVEGA | SDAARSAADI | VFLAPGLSAI | IDALKTSRQI | FHRMYAYVVY |
| 790 | 800 | 810 | 820 | 830 | 840 |
| RIALSLHLEI | FLGLWLIIRN | QLLNLELIVF | IAIFADVATL | AIAYDNAPYA | MKPVKWNLPR |
| 850 | 860 | 870 | 880 | 890 | 900 |
| LWGLATIVGI | LLAIGTWIVN | TTMIAQGQNR | GIVQNFGVQD | EVLFLQISLT | ENWLIFITRC |
| 910 | 920 | 930 | 940 | 950 | 960 |
| SGPFWSSFPS | WQLSGAVLVV | DILATLFCIF | GWFKGGHQTS | IVAVIRIWMY | SFGIFCLIAG |
| 970 | 980 | 990 | 1000 | ||
| VYYILSESSS | FDRWMHGKHK | ERGTTRKLED | FVMQLQRTST | HHEAEGKVTS |