P26359
Gene name |
msh3 (swi4, SPAC8F11.03) |
Protein name |
DNA mismatch repair protein msh3 |
Names |
Mating-type switching protein swi4, MutS protein homolog 3 |
Species |
Schizosaccharomyces pombe (strain 972 / ATCC 24843) (Fission yeast) |
KEGG Pathway |
spo:SPAC8F11.03 |
EC number |
|
Protein Class |
|
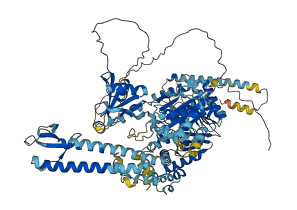
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for P26359
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-P26359-F1 | Predicted | AlphaFoldDB |
No variants for P26359
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for P26359 | |||||
No associated diseases with P26359
5 regional properties for P26359
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | DNA mismatch repair protein MutS, C-terminal | 752 - 949 | IPR000432 |
| domain | DNA mismatch repair protein MutS-like, N-terminal | 104 - 216 | IPR007695 |
| domain | DNA mismatch repair protein MutS, core | 407 - 735 | IPR007696 |
| domain | DNA mismatch repair protein MutS, connector domain | 233 - 387 | IPR007860 |
| domain | DNA mismatch repair protein MutS, clamp | 577 - 663 | IPR007861 |
3 GO annotations of cellular component
| Name | Definition |
|---|---|
| nuclear chromosome | A chromosome that encodes the nuclear genome and is found in the nucleus of a eukaryotic cell during the cell cycle phases when the nucleus is intact. |
| nucleus | A membrane-bounded organelle of eukaryotic cells in which chromosomes are housed and replicated. In most cells, the nucleus contains all of the cell's chromosomes except the organellar chromosomes, and is the site of RNA synthesis and processing. In some species, or in specialized cell types, RNA metabolism or DNA replication may be absent. |
| site of double-strand break | A region of a chromosome at which a DNA double-strand break has occurred. DNA damage signaling and repair proteins accumulate at the lesion to respond to the damage and repair the DNA to form a continuous DNA helix. |
5 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| ATP-dependent DNA damage sensor activity | A molecule that recognises toxic DNA structures, and initiates a signalling response, driven by ATP hydrolysis. |
| double-strand/single-strand DNA junction binding | Binding to a DNA segment that contains double-stranded DNA flanked by a region of single-stranded DNA. |
| double-stranded DNA binding | Binding to double-stranded DNA. |
| mismatched DNA binding | Binding to a double-stranded DNA region containing one or more mismatches. |
6 GO annotations of biological process
| Name | Definition |
|---|---|
| DNA repair | The process of restoring DNA after damage. Genomes are subject to damage by chemical and physical agents in the environment (e.g. UV and ionizing radiations, chemical mutagens, fungal and bacterial toxins, etc.) and by free radicals or alkylating agents endogenously generated in metabolism. DNA is also damaged because of errors during its replication. A variety of different DNA repair pathways have been reported that include direct reversal, base excision repair, nucleotide excision repair, photoreactivation, bypass, double-strand break repair pathway, and mismatch repair pathway. |
| gene conversion at mating-type locus | The conversion of the mating-type locus from one allele to another resulting from the recombinational repair of a site-specific double-strand break at the mating-type locus with information from a silent donor sequence. There is no reciprocal exchange of information because the mating-type locus copies information from the donor sequence and the donor sequence remains unchanged. |
| maintenance of DNA repeat elements | Any process involved in sustaining the fidelity and copy number of DNA repeat elements. |
| mismatch repair | A system for the correction of errors in which an incorrect base, which cannot form hydrogen bonds with the corresponding base in the parent strand, is incorporated into the daughter strand. The mismatch repair system promotes genomic fidelity by repairing base-base mismatches, insertion-deletion loops and heterologies generated during DNA replication and recombination. |
| mitotic recombination | The exchange, reciprocal or nonreciprocal, of genetic material between one DNA molecule and a homologous DNA region that occurs during mitotic cell cycles. |
| reciprocal meiotic recombination | The cell cycle process in which double strand breaks are formed and repaired through a single or double Holliday junction intermediate. This results in the equal exchange of genetic material between non-sister chromatids in a pair of homologous chromosomes. These reciprocal recombinant products ensure the proper segregation of homologous chromosomes during meiosis I and create genetic diversity. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MRGMSYNITH | ECDAINILSD | NLHEGAISED | MVALSGPAIE | LLENNVGSSK | NSYQEDEGSS |
| 70 | 80 | 90 | 100 | 110 | 120 |
| SIDENAPLIS | IKRKRRIRTV | KSTSNKELVQ | RKASKPTKQK | SVFTPLEQQY | LELKKNYQET |
| 130 | 140 | 150 | 160 | 170 | 180 |
| ILAIEVGYKF | RFFGKDAKIA | SEVLGISCYF | EHNFLNASVP | SYRIDYHLER | LINFGLKVAV |
| 190 | 200 | 210 | 220 | 230 | 240 |
| VRQTETAALK | STSSSRNTLF | DRRVARVLTK | GTTLDDSFFR | FEQTQHGTLQ | ASQFILCVAD |
| 250 | 260 | 270 | 280 | 290 | 300 |
| NVDKSKAKSG | RVQVGLIAIQ | LSSGTTVYDH | FQDDFLRSEL | QTRLSHFQPC | ELIYSNKLSS |
| 310 | 320 | 330 | 340 | 350 | 360 |
| ESVALLNHYV | STEKTCGRVV | RVQHAVQQDV | KLALENLQDF | FSSKCIMSGS | KIIELHMEKV |
| 370 | 380 | 390 | 400 | 410 | 420 |
| KSLHSLSIIC | LDMAISYLME | FSLEDLFVAS | NFYQPFDSIS | SMVLSKQALE | GLELFVNQTD |
| 430 | 440 | 450 | 460 | 470 | 480 |
| HTPVGSLFWV | LDRTYTRFGQ | RMLQRWLQKP | LVDKENIIER | LDAVEELAFN | SNSQVQAIRK |
| 490 | 500 | 510 | 520 | 530 | 540 |
| MLYRLPDLEK | GLSRIYYQRG | FYKAASAFSK | NSYSCFKSAL | LRRLIQQLPS | ISSIIDHFLG |
| 550 | 560 | 570 | 580 | 590 | 600 |
| MFDQKEAENN | NKVDMFKDID | NFDLSEEPND | VDYELAQEIR | ELKMSILMVR | TEMDFHLQEL |
| 610 | 620 | 630 | 640 | 650 | 660 |
| RDYLEYPNLE | FSIWGNVKFC | IEVSKGCKKI | PPDWIKLSST | RSLFRFHTPK | IQSLLIELSS |
| 670 | 680 | 690 | 700 | 710 | 720 |
| HEENLTISSE | KIYRSFLSRI | SEHYNELRNV | TTVLGTLDCL | ISFARISSQS | GYTRPEFSDK |
| 730 | 740 | 750 | 760 | 770 | 780 |
| ELLIHESRHP | MIELLSDKSF | VPNHIHLSSD | GVRCLLITGP | NMGGKSSFVK | QLALSAIMAQ |
| 790 | 800 | 810 | 820 | 830 | 840 |
| SGCFVPAKSA | LLPIFDSILI | RMGSSDNLSV | NMSTFMVEML | ETKEVLSKAT | EKSMVIIDEL |
| 850 | 860 | 870 | 880 | 890 | 900 |
| GRGTSTIDGE | AISYAVLHYL | NQYIKSYLLF | VTHFPSLGIL | ERRFEGQLRC | FHMGYLKSKE |
| 910 | 920 | 930 | 940 | 950 | 960 |
| DFETSVSQSI | SFLYKLVPGV | ASKSYGLNVA | RMAGIPFSIL | SRATEISENY | EKKHRNARKN |
| 970 | 980 | 990 | |||
| VFIRKVAKLL | MILNAEEIDF | KRLFYDLTAF | EEI |