P09880
Gene name |
TRL1 (RLG1, YJL087C, J0927) |
Protein name |
tRNA ligase |
Names |
|
Species |
Saccharomyces cerevisiae (strain ATCC 204508 / S288c) (Baker's yeast) |
KEGG Pathway |
sce:YJL087C |
EC number |
6.5.1.3: Forming phosphoric ester bonds |
Protein Class |
|
Descriptions
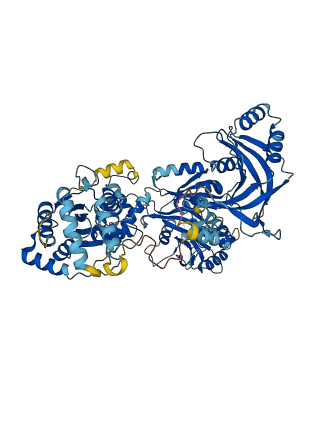
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for P09880
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-P09880-F1 | Predicted | AlphaFoldDB |
17 variants for P09880
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| s10-272228 | 85 | D>N | No | SGRP | |
| s10-272186 | 99 | N>D | No | SGRP | |
| s10-272096 | 129 | T>S | No | SGRP | |
| s10-271798 | 228 | A>V | No | SGRP | |
| s10-271787 | 232 | G>R | No | SGRP | |
| s10-271472 | 337 | K>E | No | SGRP | |
| s10-271430 | 351 | L>M | No | SGRP | |
| s10-271068 | 471 | N>K | No | SGRP | |
| s10-270972 | 503 | I>M | No | SGRP | |
| s10-270844 | 546 | K>I | No | SGRP | |
| s10-270795 | 562 | Q>H | No | SGRP | |
| s10-270700 | 594 | I>T | No | SGRP | |
| s10-270521 | 654 | E>Q | No | SGRP | |
| s10-270479 | 668 | V>I | No | SGRP | |
| s10-270195 | 762 | N>K | No | SGRP | |
| s10-270101 | 794 | V>I | No | SGRP | |
| s10-270050 | 811 | V>L | No | SGRP |
No associated diseases with P09880
No regional properties for P09880
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| No domain, repeats, and functional sites for P09880 | |||
Functions
| Description | ||
|---|---|---|
| EC Number | 6.5.1.3 | Forming phosphoric ester bonds |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
2 GO annotations of cellular component
| Name | Definition |
|---|---|
| cytoplasm | The contents of a cell excluding the plasma membrane and nucleus, but including other subcellular structures. |
| nuclear inner membrane | The inner, i.e. lumen-facing, lipid bilayer of the nuclear envelope. |
5 GO annotations of molecular function
| Name | Definition |
|---|---|
| 2',3'-cyclic-nucleotide 3'-phosphodiesterase activity | Catalysis of the reaction: nucleoside 2',3'-cyclic phosphate + H2O = nucleoside 2'-phosphate. |
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| endonuclease activity | Catalysis of the hydrolysis of ester linkages within nucleic acids by creating internal breaks. |
| GTP-dependent polyribonucleotide 5'-hydroxyl-kinase activity | Catalysis of the reaction: GTP + 5'-dephospho-RNA = GDP + 5'-phospho-RNA. |
| RNA ligase (ATP) activity | Catalysis of the reaction: ATP + ribonucleotide(n) + ribonucleotide(m) = AMP + diphosphate + ribonucleotide(n+m). |
5 GO annotations of biological process
| Name | Definition |
|---|---|
| IRE1-mediated unfolded protein response | The series of molecular signals mediated by the endoplasmic reticulum stress sensor IRE1 (Inositol-requiring transmembrane kinase/endonuclease). Begins with activation of IRE1 in response to endoplasmic reticulum (ER) stress, and ends with regulation of a downstream cellular process, e.g. transcription. One target of activated IRE1 is the transcription factor HAC1 in yeast, or XBP1 in mammals; IRE1 cleaves an intron of a mRNA coding for HAC1/XBP1 to generate an activated HAC1/XBP1 transcription factor, which controls the up regulation of UPR-related genes. At least in mammals, IRE1 can also signal through additional intracellular pathways including JNK and NF-kappaB. |
| phosphorylation | The process of introducing a phosphate group into a molecule, usually with the formation of a phosphoric ester, a phosphoric anhydride or a phosphoric amide. |
| positive regulation of translation in response to stress | Any process that activates or increases the frequency, rate or extent of translation as a result of a stimulus indicating the organism is under stress. |
| regulation of nuclear-transcribed mRNA catabolic process, nonsense-mediated decay | Any process that modulates the frequency, rate or extent of nuclear-transcribed mRNA catabolic process, nonsense-mediated decay. |
| tRNA splicing, via endonucleolytic cleavage and ligation | Splicing of tRNA substrates via recognition of the folded RNA structure that brings the 5' and 3' splice sites into proximity and cleavage of the RNA at both the 3' and 5' splice sites by an endonucleolytic mechanism, followed by ligation of the exons. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MPSPYDGKRT | VTQLVNELEK | AEKLSGRGRA | YRRVCDLSHS | NKKVISWKFN | EWDYGKNTIT |
| 70 | 80 | 90 | 100 | 110 | 120 |
| LPCNARGLFI | SDDTTNPVIV | ARGYDKFFNV | GEVNFTKWNW | IEENCTGPYD | VTIKANGCII |
| 130 | 140 | 150 | 160 | 170 | 180 |
| FISGLEDGTL | VVCSKHSTGP | RADVDRNHAE | AGEKQLLRQL | AAMNINRSDF | ARMLYTHNVT |
| 190 | 200 | 210 | 220 | 230 | 240 |
| AVAEYCDDSF | EEHILEYPLE | KAGLYLHGVN | VNKAEFETWD | MKDVSQMASK | YGFRCVQCIT |
| 250 | 260 | 270 | 280 | 290 | 300 |
| SNTLEDLKKF | LDNCSATGSF | EGQEIEGFVI | RCHLKSTEKP | FFFKYKFEEP | YLMYRQWREV |
| 310 | 320 | 330 | 340 | 350 | 360 |
| TKDYISNKSR | VFKFRKHKFI | TNKYLDFAIP | ILESSPKICE | NYLKGFGVIE | LRNKFLQSYG |
| 370 | 380 | 390 | 400 | 410 | 420 |
| MSGLEILNHE | KVAELELKNA | IDYDKVDERT | KFLIFPISVI | GCGKTTTSQT | LVNLFPDSWG |
| 430 | 440 | 450 | 460 | 470 | 480 |
| HIQNDDITGK | DKSQLMKKSL | ELLSKKEIKC | VIVDRNNHQF | RERKQLFEWL | NELKEDYLVY |
| 490 | 500 | 510 | 520 | 530 | 540 |
| DTNIKVIGVS | FAPYDKLSEI | RDITLQRVIK | RGNNHQSIKW | DELGEKKVVG | IMNGFLKRYQ |
| 550 | 560 | 570 | 580 | 590 | 600 |
| PVNLDKSPDN | MFDLMIELDF | GQADSSLTNA | KQILNEIHKA | YPILVPEIPK | DDEIETAFRR |
| 610 | 620 | 630 | 640 | 650 | 660 |
| SLDYKPTVRK | IVGKGNNNQQ | KTPKLIKPTY | ISAKIENYDE | IIELVKRCIA | SDAELTEKFK |
| 670 | 680 | 690 | 700 | 710 | 720 |
| HLLASGKVQK | ELHITLGHVM | SSREKEAKKL | WKSYCNRYTD | QITEYNNNRI | ENAQGSGNNQ |
| 730 | 740 | 750 | 760 | 770 | 780 |
| NTQVKTTDKL | NFRLEKLCWD | EKIIAIVVEL | SKDKDGCIID | ENNEKIKGLC | CQNKIPHITL |
| 790 | 800 | 810 | 820 | ||
| CKLESGVKAV | YSNVLCEKVE | SAEVDENIKV | VKLDNSKEFV | GSVYLNF |