O93794
Gene name |
TOP2 (CAGL0J05610g) |
Protein name |
DNA topoisomerase 2 |
Names |
DNA topoisomerase II |
Species |
Candida glabrata (strain ATCC 2001 / CBS 138 / JCM 3761 / NBRC 0622 / NRRL Y-65) (Yeast) (Torulopsis glabrata) |
KEGG Pathway |
cgr:CAGL0J05610g |
EC number |
5.6.2.2: Enzymes altering nucleic acid conformation |
Protein Class |
|
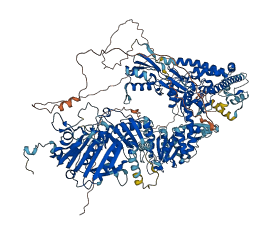
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for O93794
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-O93794-F1 | Predicted | AlphaFoldDB |
No variants for O93794
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for O93794 | |||||
No associated diseases with O93794
7 regional properties for O93794
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | DNA topoisomerase, type IIA, domain A | 668 - 1162 | IPR002205 |
| domain | Histidine kinase/HSP90-like ATPase | 57 - 204 | IPR003594 |
| domain | TOPRIM domain | 441 - 555 | IPR006171 |
| domain | DNA topoisomerase, type IIA, subunit B, domain 2 | 246 - 412 | IPR013506 |
| conserved_site | DNA topoisomerase, type IIA, conserved site | 445 - 453 | IPR018522 |
| domain | C-terminal associated domain of TOPRIM | 557 - 686 | IPR031660 |
| domain | DNA topoisomerase 2, TOPRIM domain | 441 - 559 | IPR034157 |
Functions
| Description | ||
|---|---|---|
| EC Number | 5.6.2.2 | Enzymes altering nucleic acid conformation |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
4 GO annotations of cellular component
| Name | Definition |
|---|---|
| chromosome, centromeric core domain | The innermost portion of the centromeric region of a chromosome, encompassing the core region of a chromosome centromere and the proteins that bind to it. |
| DNA replication termination region | A chromosomal region that contains fork pausing elements influencing the progression and merging of DNA replication forks. |
| euchromatin | A dispersed and relatively uncompacted form of chromatin that is in a transcription-competent conformation. |
| synaptonemal complex | A proteinaceous scaffold found between homologous chromosomes during meiosis. It consists of 2 lateral elements and a central element, all running parallel to each other. Transverse filaments connect the lateral elements to the central element. |
5 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| DNA binding | Any molecular function by which a gene product interacts selectively and non-covalently with DNA (deoxyribonucleic acid). |
| DNA topoisomerase type II (double strand cut, ATP-hydrolyzing) activity | Catalysis of a DNA topological transformation by transiently cleaving a pair of complementary DNA strands to form a gate through which a second double-stranded DNA segment is passed, after which the severed strands in the first DNA segment are rejoined, driven by ATP hydrolysis. The enzyme changes the linking number in multiples of 2. |
| identical protein binding | Binding to an identical protein or proteins. |
| metal ion binding | Binding to a metal ion. |
8 GO annotations of biological process
| Name | Definition |
|---|---|
| chromatin remodeling at centromere | Dynamic structural changes in centromeric DNA. |
| DNA strand elongation involved in DNA replication | The process in which an existing DNA strand is extended by activities including the addition of nucleotides to the 3' end of the strand, complementary to an existing template, as part of DNA replication. |
| DNA topological change | The process in which a transformation is induced in the topological structure of a double-stranded DNA helix, resulting in a change in linking number. |
| mitotic chromosome condensation | The cell cycle process in which chromatin structure is compacted prior to and during mitosis in eukaryotic cells. |
| regulation of mitotic recombination | Any process that modulates the frequency, rate or extent of DNA recombination during mitosis. |
| replication fork progression beyond termination site | Regulation of DNA replication by a mechanism that allows a DNA replication fork to progress beyond a termination site, which is a region containing fork pausing elements that influence the progression and merging of DNA replication forks. |
| resolution of meiotic recombination intermediates | The cleavage and rejoining of intermediates, such as Holliday junctions, formed during meiotic recombination to produce two intact molecules in which genetic material has been exchanged. |
| rRNA transcription | The synthesis of ribosomal RNA (rRNA), any RNA that forms part of the ribosomal structure, from a DNA template. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MSEPKTASER | YQKISQLEHI | LKRPDTYIGS | VEIQEQEQWI | YDEETDCMID | KTVNIVPGLF |
| 70 | 80 | 90 | 100 | 110 | 120 |
| KIFDEILVNA | ADNKVRDPSM | KRIDVTINPE | ENFIEVRNDG | KGIPIEIHEK | EKIYIPELIF |
| 130 | 140 | 150 | 160 | 170 | 180 |
| GHLLTSSNYD | DDEKKVTGGR | NGYGAKLCNI | FSTEFTLETA | DPKNGRKYVQ | TWENNMNVCH |
| 190 | 200 | 210 | 220 | 230 | 240 |
| PPKITSYKKG | PSYTKVAFKP | DLSRFGMESL | DSDILGVMRR | RVYDINGSVR | DVNVYLNGKP |
| 250 | 260 | 270 | 280 | 290 | 300 |
| LKIRNFKNYV | ELYLKSLEKM | RKMDNGESDT | TPSNIPTILY | ERVSDRWEIA | FAVSDISFKQ |
| 310 | 320 | 330 | 340 | 350 | 360 |
| VSFVNSIATT | TGGTHVNYIA | DQIVRKVSDI | LKKKKKNIKP | YQIKNNMFIF | INCLIENPAF |
| 370 | 380 | 390 | 400 | 410 | 420 |
| TSQTKEQLTT | RVKDFGSRCD | ISSDYINKIM | KTDLATKIFE | IADENANNAL | KKSDGSRKSR |
| 430 | 440 | 450 | 460 | 470 | 480 |
| ITDYPKLEDA | NKAGTKDGYK | CTLILTEGDS | ALSLAVAGLA | VVGRDYYGCY | PLRGKMLNVR |
| 490 | 500 | 510 | 520 | 530 | 540 |
| EATADQILKN | AEIQAIKKIM | GLQHRKKYED | TKSLRYGHLM | IMTDQDHDGS | HIKGLIINFI |
| 550 | 560 | 570 | 580 | 590 | 600 |
| ETSFPGLLDI | PGFLIEFITP | IVKVTITKPI | KKVISFFNLP | DYEKWREEES | HKYSWKQKYY |
| 610 | 620 | 630 | 640 | 650 | 660 |
| KGLGTSTSPE | IIEYFSNLDT | HLKKFHALQG | DDKDLIDLAF | SKKKADDRKE | WLRQYEPGTV |
| 670 | 680 | 690 | 700 | 710 | 720 |
| LDPTLNEIPI | SDFINKELIL | FSLADNVRSI | PSVLDGFKPG | QRKVLYTCFK | KNLTTEKKVA |
| 730 | 740 | 750 | 760 | 770 | 780 |
| NLAPAVSDYT | AYHHGEQALV | QTIIGMAQNF | VGTNNIYFLK | PNGAFGTRAT | GGKDAAAARY |
| 790 | 800 | 810 | 820 | 830 | 840 |
| IYTELNKIAR | KVFHPADDPL | FRYVQEDEKT | VEPEWYLPVV | PMVLINGAEG | IGTGWSTSIP |
| 850 | 860 | 870 | 880 | 890 | 900 |
| PFNPLDVVNN | IRHLLNDEEM | DDMHPWFRGW | TGTMEKIESQ | RYRMYGRIEQ | VGPNTLEITE |
| 910 | 920 | 930 | 940 | 950 | 960 |
| LPARTWTSTI | KEHLLLGLGG | SEKVKPWIKD | MEEQHAETIK | FIIKLTDEEM | TKTRKLGFYE |
| 970 | 980 | 990 | 1000 | 1010 | 1020 |
| RFKLISPISL | QNMVAFDYRG | KIKKYDHVHE | ILKDFYEVRL | EYYQKRKDYM | TGRLQWEAEK |
| 1030 | 1040 | 1050 | 1060 | 1070 | 1080 |
| LSFQVKFIKM | IIDKSLIVTN | KPKKQLISEL | EELGFPRINK | EGKPHFGKID | EEVEAIISED |
| 1090 | 1100 | 1110 | 1120 | 1130 | 1140 |
| EDEDLEESEE | ATRKKDKDDE | STVNGPEELF | GTYEYLLGLK | IWSLTKERYE | KLLKQKQEKE |
| 1150 | 1160 | 1170 | 1180 | 1190 | 1200 |
| TELENLLKLS | AKDLWNNDLD | DFLTAYEDFQ | KMDLFLRNSA | VPKTKGGKRK | RKGGDDDDYD |
| 1210 | 1220 | 1230 | 1240 | 1250 | 1260 |
| PSGKKKPARR | IKKIKKEDDF | DRILIKPQAK | IKAKRPVKVK | VEPPSSAAST | PSVKEELGVS |
| 1270 | 1280 | 1290 | 1300 | 1310 | 1320 |
| DVTSNASTPS | TTIFDQKVKQ | ENSDESGISA | FSSKFNKIAS | AFDEDAPLDQ | ITSEDTSVKE |
| 1330 | 1340 | 1350 | 1360 | 1370 | 1380 |
| SSAPAAKKKA | PPKRKAKVVE | SSEDELSDAN | LSEQDDEEVV | PVRRQRSSRQ | TAKKSYAEPI |
| 1390 | 1400 | ||||
| EISDEEDFID | DDEDEEVDSD | ESFNDE |