O74475
Gene name |
bgs4 (SPCC1840.02c) |
Protein name |
1,3-beta-glucan synthase component bgs4 |
Names |
1,3-beta-D-glucan-UDP glucosyltransferase |
Species |
Schizosaccharomyces pombe (strain 972 / ATCC 24843) (Fission yeast) |
KEGG Pathway |
spo:SPCC1840.02c |
EC number |
2.4.1.34: Hexosyltransferases |
Protein Class |
|
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
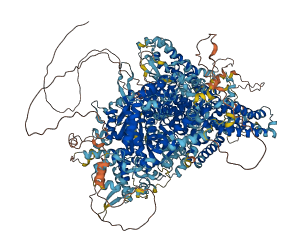
1 structures for O74475
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-O74475-F1 | Predicted | AlphaFoldDB |
No variants for O74475
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for O74475 | |||||
No associated diseases with O74475
1 regional properties for O74475
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | 1,3-beta-glucan synthase component FKS1-like, domain-1 | 363 - 475 | IPR026899 |
Functions
| Description | ||
|---|---|---|
| EC Number | 2.4.1.34 | Hexosyltransferases |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
14 GO annotations of cellular component
| Name | Definition |
|---|---|
| 1,3-beta-D-glucan synthase complex | A protein complex that catalyzes the transfer of a glucose group from UDP-glucose to a (1->3)-beta-D-glucan chain. |
| cell division site | The eventual plane of cell division (also known as cell cleavage or cytokinesis) in a dividing cell. In Eukaryotes, the cleavage apparatus, composed of septin structures and the actomyosin contractile ring, forms along this plane, and the mitotic, or meiotic, spindle is aligned perpendicular to the division plane. In bacteria, the cell division site is generally located at mid-cell and is the site at which the cytoskeletal structure, the Z-ring, assembles. |
| cell tip | The region at the end of the longest axis of a cylindrical or elongated cell. |
| cleavage furrow | The cleavage furrow is a plasma membrane invagination at the cell division site. The cleavage furrow begins as a shallow groove and eventually deepens to divide the cytoplasm. |
| cytoplasm | The contents of a cell excluding the plasma membrane and nucleus, but including other subcellular structures. |
| division septum | A cell septum which forms as part of the division site and functions in the compartmentalization of a cell into two daughter cells at division. A division septum spans a cell and does not allow exchange of organelles or cytoplasm between compartments. |
| Golgi apparatus | A membrane-bound cytoplasmic organelle of the endomembrane system that further processes the core oligosaccharides (e.g. N-glycans) added to proteins in the endoplasmic reticulum and packages them into membrane-bound vesicles. The Golgi apparatus operates at the intersection of the secretory, lysosomal, and endocytic pathways. |
| integral component of membrane | The component of a membrane consisting of the gene products and protein complexes having at least some part of their peptide sequence embedded in the hydrophobic region of the membrane. |
| mating projection tip | The apex of the mating projection in unicellular fungi exposed to mating pheromone; site of polarized growth. |
| new growing cell tip | A cell tip that was newly formed at the last cell division, and that has started to grow after the cell has activated bipolar cell growth (i.e. in which new end take-off, NETO, has taken place). New end take-off is when monopolar cells initiate bipolar growth. |
| plasma membrane | The membrane surrounding a cell that separates the cell from its external environment. It consists of a phospholipid bilayer and associated proteins. |
| plasma membrane of cell tip | The portion of the plasma membrane surrounding the cell tip. |
| primary cell septum | A cell septum that forms following nuclear division. |
| site of polarized growth | Any part of a cell where non-isotropic growth takes place. |
2 GO annotations of molecular function
| Name | Definition |
|---|---|
| 1,3-beta-D-glucan synthase activity | Catalysis of the reaction: UDP-glucose + [(1->3)-beta-D-glucosyl](n) = UDP + [(1->3)-beta-D-glucosyl](n+1). |
| glucosyltransferase activity | Catalysis of the transfer of a glucosyl group to an acceptor molecule, typically another carbohydrate or a lipid. |
4 GO annotations of biological process
| Name | Definition |
|---|---|
| (1->3)-beta-D-glucan biosynthetic process | The chemical reactions and pathways resulting in the formation of (1->3)-beta-D-glucans, compounds composed of glucose residues linked by (1->3)-beta-D-glucosidic bonds. |
| fungal-type cell wall (1->3)-beta-D-glucan biosynthetic process | The chemical reactions and pathways resulting in the formation of (1->3)-beta-D-glucans, compounds composed of glucose residues linked by (1->3)-beta-D-glucosidic bonds, found in fungal cell walls. |
| fungal-type cell wall polysaccharide biosynthetic process | The chemical reactions and pathways resulting in the formation of the polysaccharides which make up the fungal-type cell wall. |
| secondary cell septum biogenesis | A cellular process that results in the biosynthesis of constituent macromolecules, assembly, and arrangement of constituent parts of a secondary cell septum following nuclear division. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MSGNNENVSG | ITGHDAVSDD | QYAYDSEVYD | DQNAYQRQPA | DAYSNEEFLD | QADYDSMYGE |
| 70 | 80 | 90 | 100 | 110 | 120 |
| GYNGYDYPTG | VTESYGDEYT | PVDTASSGIN | QYSTEKGKFT | RPSDEYESEY | SDYNAQPSDA |
| 130 | 140 | 150 | 160 | 170 | 180 |
| NNFYNLRGDG | RYNAYDPSSD | SLANVYNSVP | YGSSPYDFSN | SSFVGNSGSG | TPLDGDSGSF |
| 190 | 200 | 210 | 220 | 230 | 240 |
| YADSANLTNR | EPYPAWTPEN | ELPLTKEEIE | DIFIDLTNKL | GFQRDSMRNM | YDFFMCLLDS |
| 250 | 260 | 270 | 280 | 290 | 300 |
| RASRMTPDQA | LLTLHADYIG | SDIANYKKWY | FASQMDREDA | VGLANVGIYG | GKVTSIKEKG |
| 310 | 320 | 330 | 340 | 350 | 360 |
| KFFSRNKKAP | KVVKPPRKSR | FKRKKKKEQP | EEAEDEYIDV | NTDDSLESAE | YRWRSHMRSM |
| 370 | 380 | 390 | 400 | 410 | 420 |
| TQFERAQQIA | LWLLLWGEAN | NVRFMPEVIA | FLFKCAYDYI | ISPEAQNVTE | PVPEGYYLDN |
| 430 | 440 | 450 | 460 | 470 | 480 |
| IVSPLYQYMH | DQQFEIINGK | YVRRERPHDQ | LIGYDDINQL | FWHAEGIARL | IFEDGTRLID |
| 490 | 500 | 510 | 520 | 530 | 540 |
| IPASERFHRL | PEVQWNRAFY | KTYYESRSWF | HLITNFNRIW | VIHFGMFWYF | TAFNSPTLYT |
| 550 | 560 | 570 | 580 | 590 | 600 |
| KPFHQRDGPK | PTGASQWAAV | ACTSVVSCII | MAAASLCEYL | FVPRRFPGSK | PIWKRLCIIV |
| 610 | 620 | 630 | 640 | 650 | 660 |
| LIAIINLIPI | VYIFGFSSKH | QQRSGRRIAV | GVVAFLMSIA | TYVYFSLVPL | QSTFGKLSVK |
| 670 | 680 | 690 | 700 | 710 | 720 |
| DSRKYLANKY | FTSNFAPLKF | DNQALSVIIW | VCVFTCKFAE | SYFFLTLSIR | DPIIVLSTMR |
| 730 | 740 | 750 | 760 | 770 | 780 |
| PYLCSIYWAG | SRLCFVQPRI | ILGIMYFTDL | ILFFLDTYLW | YIIFNTIFSV | LRSFVLGISI |
| 790 | 800 | 810 | 820 | 830 | 840 |
| LTPWRNIFSR | MPQRIYGKIL | ATNDMEIKYK | PKILISQIWN | AIVISMYREH | LLSIDHVQRL |
| 850 | 860 | 870 | 880 | 890 | 900 |
| LYHQVPAEEG | RRTLRTPTFF | VSQDDNIVHT | TFFPANSEAE | RRLSFFAQSL | ATPIPEPVPV |
| 910 | 920 | 930 | 940 | 950 | 960 |
| DNMPTFTVLI | PHYAEKILLS | LREIIREEDQ | LSRVTLLEYL | KQLHPVEWDC | FVKDTKILVE |
| 970 | 980 | 990 | 1000 | 1010 | 1020 |
| ENAPYENDSV | SEKEGTYKSK | VDDLPFYCIG | FKSAMPEYTL | RTRIWASLRS | QTLYRTISGF |
| 1030 | 1040 | 1050 | 1060 | 1070 | 1080 |
| MNYSRAIKLL | YRVENPEIVQ | MFGGNTDRLE | RELDRMARRK | FKLVVSMQRY | AKFTKEEYEN |
| 1090 | 1100 | 1110 | 1120 | 1130 | 1140 |
| AEFLLRAYPD | LQIAYLDEDP | PEEEGAEPQL | FAALIDGHSE | IMENERRRPK | YRIRLSGNPI |
| 1150 | 1160 | 1170 | 1180 | 1190 | 1200 |
| LGDGKSDNQN | MSLPFYRGEY | IQLIDANQDN | YLEECLKIRS | VLAEFEEMET | DNVNPYSESA |
| 1210 | 1220 | 1230 | 1240 | 1250 | 1260 |
| RERNKHPVAI | LGAREYIFSE | NIGILGDVAA | GKEQTFGTLF | SRTLAQIGGK | LHYGHPDFLN |
| 1270 | 1280 | 1290 | 1300 | 1310 | 1320 |
| GIFMTTRGGV | SKAQKGLHVN | EDIYAGMNAM | LRGGRIKHCE | YFQCGKGRDL | GFGSILNFNT |
| 1330 | 1340 | 1350 | 1360 | 1370 | 1380 |
| KVGTGMGEQM | LSREYYYLGT | QLQLDRFLSF | YFAHPGFHLN | NMFIMLSVQL | FMVVLINLGA |
| 1390 | 1400 | 1410 | 1420 | 1430 | 1440 |
| IYHVVTVCYY | NGNQKLSYDT | SIVPRGCYQL | GPVLSWLKRC | VISIFIVFWI | SFIPLTVHEL |
| 1450 | 1460 | 1470 | 1480 | 1490 | 1500 |
| IERGVWRATK | RFFKQIGSFS | PLFEVFTCQV | YSQAITSDLA | YGGARYIGTG | RGFATARLPF |
| 1510 | 1520 | 1530 | 1540 | 1550 | 1560 |
| SILYSRFAVP | SIYIGARFLM | MLLFGTMTVW | VAHLIYWWVS | IMALCVAPFL | FNPHQFDWND |
| 1570 | 1580 | 1590 | 1600 | 1610 | 1620 |
| FFVDYREFIR | WLSRGNSRSH | ANSWIGYCRL | TRTRITGYKR | RVLGQPSDKI | SMDTPRAKFT |
| 1630 | 1640 | 1650 | 1660 | 1670 | 1680 |
| NVFFSDVLIP | ALLAAGAIIP | YFFINSQPGN | PMFITDPNNP | SPYVHDTKTG | TNPILRLVII |
| 1690 | 1700 | 1710 | 1720 | 1730 | 1740 |
| SLIPIAAGFG | MSGFFGGMAC | CLGPAFGLCC | KKFPSIFAAI | AHTIQIFIFI | AIFEVCWFLD |
| 1750 | 1760 | 1770 | 1780 | 1790 | 1800 |
| GWSLPKTVLA | FCAVTAIHRF | IFKILTLLCL | SREVKQDSAN | ISWWSGKWYG | KGYGYHAFTL |
| 1810 | 1820 | 1830 | 1840 | 1850 | 1860 |
| PAREFVCKAI | ELNLFATDFF | LGHLLLFFML | PVICIPYIDR | WHSVLLFWLR | PSRQIRPPIF |
| 1870 | 1880 | 1890 | 1900 | 1910 | 1920 |
| STKQNRLRKR | IVRRYSALYF | SILVIFLILI | IVPLAAGAEI | RQGLTASEAV | AKGAVGWNQT |
| 1930 | 1940 | 1950 | |||
| NSSIGSGIIQ | PRDTNYTANY | SFWYDRYHFE | FNTTY |