O59824
Gene name |
SPCC965.04c |
Protein name |
ATP-dependent zinc metalloprotease YME1 homolog |
Names |
|
Species |
Schizosaccharomyces pombe (strain 972 / ATCC 24843) (Fission yeast) |
KEGG Pathway |
spo:SPCC965.04c |
EC number |
|
Protein Class |
|
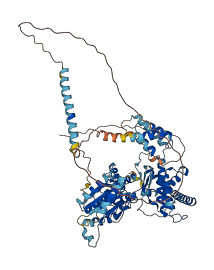
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for O59824
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-O59824-F1 | Predicted | AlphaFoldDB |
No variants for O59824
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for O59824 | |||||
No associated diseases with O59824
4 GO annotations of cellular component
| Name | Definition |
|---|---|
| i-AAA complex | Protease complex of the mitochondrial inner membrane whose catalytic residues lie on the intermembrane space side of the inner membrane; involved in mitochondrial protein turnover. Contains a subunit belonging to the AAA family of ATP-dependent metalloproteases. |
| integral component of membrane | The component of a membrane consisting of the gene products and protein complexes having at least some part of their peptide sequence embedded in the hydrophobic region of the membrane. |
| mitochondrial inner membrane | The inner, i.e. lumen-facing, lipid bilayer of the mitochondrial envelope. It is highly folded to form cristae. |
| mitochondrion | A semiautonomous, self replicating organelle that occurs in varying numbers, shapes, and sizes in the cytoplasm of virtually all eukaryotic cells. It is notably the site of tissue respiration. |
5 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| ATP hydrolysis activity | Catalysis of the reaction: ATP + H2O = ADP + H+ phosphate. ATP hydrolysis is used in some reactions as an energy source, for example to catalyze a reaction or drive transport against a concentration gradient. |
| ATP-dependent peptidase activity | Catalysis of the hydrolysis of peptide bonds, driven by ATP hydrolysis. |
| metal ion binding | Binding to a metal ion. |
| metalloendopeptidase activity | Catalysis of the hydrolysis of internal, alpha-peptide bonds in a polypeptide chain by a mechanism in which water acts as a nucleophile, one or two metal ions hold the water molecule in place, and charged amino acid side chains are ligands for the metal ions. |
4 GO annotations of biological process
| Name | Definition |
|---|---|
| mitochondrial protein catabolic process | The chemical reactions and pathways resulting in the breakdown of a mitochondrial protein. This process is necessary to maintain the healthy state of mitochondria and is thought to occur via the induction of an intramitochondrial lysosome-like organelle that acts to eliminate the damaged oxidised mitochondrial proteins without destroying the mitochondrial structure. |
| mitochondrion organization | A process that is carried out at the cellular level which results in the assembly, arrangement of constituent parts, or disassembly of a mitochondrion; includes mitochondrial morphogenesis and distribution, and replication of the mitochondrial genome as well as synthesis of new mitochondrial components. |
| protein quality control for misfolded or incompletely synthesized proteins | The chemical reactions and pathways resulting in the breakdown of misfolded or attenuated proteins. |
| proteolysis | The hydrolysis of proteins into smaller polypeptides and/or amino acids by cleavage of their peptide bonds. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MSRVLHPIFL | FGKTSFLYSG | CSKFGGRLFN | NSIVHGWLRT | RSYALASGLH | PLRKQKLAHF |
| 70 | 80 | 90 | 100 | 110 | 120 |
| EDLANANMSD | PYMQAKLYKE | LADNFPEAII | SRYETQGVAR | NSACDRYYQE | ALRKKSWSRS |
| 130 | 140 | 150 | 160 | 170 | 180 |
| LSNNISLSQS | SSSPATSSFS | DPKAFSAGVP | KFTSDTSSTV | SSTPSLNHSL | QNSMPPSTPT |
| 190 | 200 | 210 | 220 | 230 | 240 |
| PPPVWAPTIV | SSALGTSSKT | PVYVVVDEPR | FTKFFRIFKF | IAGLSVASYF | VLLGMSIFAE |
| 250 | 260 | 270 | 280 | 290 | 300 |
| TSGLNNIMTN | TTEQEPMEER | AINVRFSDVQ | GVDEAKEELE | EIVDFLRDPT | HFTRLGGKLP |
| 310 | 320 | 330 | 340 | 350 | 360 |
| RGVLLTGPPG | TGKTMLARAV | AGEANVPFFF | MSGSQFDEMY | VGVGAKRVRE | LFAAARKQAP |
| 370 | 380 | 390 | 400 | 410 | 420 |
| SIIFIDELDA | IGQKRNARDA | AHMRQTLNQL | LVDLDGFSKN | EDLAHPVVFI | GATNFPESLD |
| 430 | 440 | 450 | 460 | 470 | 480 |
| PALTRPGRFD | RHIHVPLPDV | RGRLAILLQH | TRHVPLGKDV | DLSIIARGTS | GFAGADLANL |
| 490 | 500 | 510 | 520 | 530 | 540 |
| INQAAVYASK | NLSTAVSMRD | LEWSKDRILM | GAERKSAFIT | PENKLMTAYH | EGGHALVALF |
| 550 | 560 | 570 | 580 | 590 | 600 |
| TKNAMRPYKA | TIMPRGSSLG | MTISLPDMDK | DSWTREEYLA | MLDVTMGGRA | AEELLYGKDK |
| 610 | 620 | 630 | 640 | 650 | 660 |
| ITSGAHNDID | KATQVARRMV | TEFGMSDRIG | PVSLEAEMDN | LSPATRALVE | SEIKSLLEAS |
| 670 | 680 | 690 | 700 | ||
| YERSLSLLKS | HKKELDALAT | ALVDYEFLTA | EEMNRVVKGD | RDLLRNKLS |