O54956
Gene name |
Pole2 |
Protein name |
DNA polymerase epsilon subunit 2 |
Names |
DNA polymerase II subunit 2, DNA polymerase epsilon subunit B |
Species |
Mus musculus (Mouse) |
KEGG Pathway |
mmu:18974 |
EC number |
|
Protein Class |
|
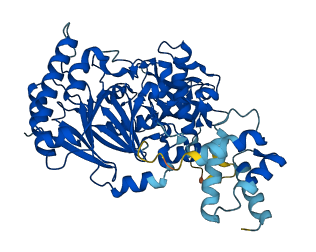
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for O54956
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-O54956-F1 | Predicted | AlphaFoldDB |
26 variants for O54956
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| rs29135637 | 78 | M>V | No | EVA | |
| rs3389243667 | 87 | N>Y | No | EVA | |
| rs3389209538 | 112 | T>P | No | EVA | |
| rs236242260 | 115 | A>T | No | EVA | |
| rs3389238593 | 116 | A>V | No | EVA | |
| rs3389227676 | 133 | R>H | No | EVA | |
| rs3389249819 | 145 | E>D | No | EVA | |
| rs3389240843 | 145 | E>G | No | EVA | |
| rs3389237041 | 155 | H>Y | No | EVA | |
| rs3389252168 | 157 | E>V | No | EVA | |
| rs3389200903 | 182 | I>M | No | EVA | |
| rs3389255520 | 195 | F>C | No | EVA | |
| rs3389173019 | 201 | T>N | No | EVA | |
| rs3389237025 | 203 | T>I | No | EVA | |
| rs3403499844 | 205 | Q>E | No | EVA | |
| rs3402692676 | 205 | Q>L | No | EVA | |
| rs3389215946 | 206 | L>M | No | EVA | |
| rs3389200873 | 212 | Q>H | No | EVA | |
| rs3389238632 | 245 | T>A | No | EVA | |
| rs3389237026 | 333 | N>Y | No | EVA | |
| rs3389200869 | 376 | L>I | No | EVA | |
| rs3403006821 | 390 | R>* | No | EVA | |
| rs3402692678 | 457 | Y>* | No | EVA | |
| rs3403006875 | 458 | V>I | No | EVA | |
| rs3403377681 | 459 | C>* | No | EVA | |
| rs3403519887 | 470 | R>N | No | EVA |
No associated diseases with O54956
4 GO annotations of cellular component
| Name | Definition |
|---|---|
| epsilon DNA polymerase complex | A heterotetrameric DNA polymerase complex that catalyzes processive DNA synthesis in the absence of PCNA, but is further stimulated in the presence of PCNA. The complex contains a large catalytic subunit and three small subunits, and is best characterized in Saccharomyces, in which the subunits are named Pol2p, Dpb2p, Dpb3p, and Dpb4p. Some evidence suggests that DNA polymerase epsilon is the leading strand polymerase; it is also involved in nucleotide-excision repair and mismatch repair. |
| intracellular membrane-bounded organelle | Organized structure of distinctive morphology and function, bounded by a single or double lipid bilayer membrane and occurring within the cell. Includes the nucleus, mitochondria, plastids, vacuoles, and vesicles. Excludes the plasma membrane. |
| nuclear body | Extra-nucleolar nuclear domains usually visualized by confocal microscopy and fluorescent antibodies to specific proteins. |
| nucleoplasm | That part of the nuclear content other than the chromosomes or the nucleolus. |
1 GO annotations of molecular function
| Name | Definition |
|---|---|
| DNA binding | Any molecular function by which a gene product interacts selectively and non-covalently with DNA (deoxyribonucleic acid). |
2 GO annotations of biological process
| Name | Definition |
|---|---|
| DNA-templated DNA replication | A DNA replication process that uses parental DNA as a template for the DNA-dependent DNA polymerases that synthesize the new strands. |
| error-prone translesion synthesis | The conversion of DNA-damage induced single-stranded gaps into large molecular weight DNA after replication by using a specialized DNA polymerase or replication complex to insert a defined nucleotide across the lesion. This process does not remove the replication-blocking lesions and causes an increase in the endogenous mutation level. For example, in E. coli, a low fidelity DNA polymerase, pol V, copies lesions that block replication fork progress. This produces mutations specifically targeted to DNA template damage sites, but it can also produce mutations at undamaged sites. |
| 10 | 20 | 30 | 40 | 50 | 60 |
| MAPERLRSRT | VSAFKLRGLL | LRSEATKYLT | EALQSVTELE | LEENLGKIID | AVEKQPLSSN |
| 70 | 80 | 90 | 100 | 110 | 120 |
| MIERSVVEAA | VQECSQSMDE | TIEHVFNIIG | AFDIPRFIYN | SERKKFLPLS | MTNHAAPTLF |
| 130 | 140 | 150 | 160 | 170 | 180 |
| GTARDKAELY | LERYTILHQR | THRHELFTPP | VIGSHLEESG | SKFQLKTIET | LLGSTSKVGD |
| 190 | 200 | 210 | 220 | 230 | 240 |
| VIVLGMITQL | KEGKFFLEDP | TGTVQLDLSK | AQFHSGLYTE | ACFVLAEGWF | EDQVFHANAF |
| 250 | 260 | 270 | 280 | 290 | 300 |
| GFPPTEPSST | TRAYYGNINF | FGGPSNASVK | TYTKLRQLED | ENKDAMFVIV | SDVWLDQVQV |
| 310 | 320 | 330 | 340 | 350 | 360 |
| LEKFHVMFSG | YSPAPPTCFI | LCGNFSSAPY | GKNQVQALKD | SLKSLADIIC | EYPSIHQSSR |
| 370 | 380 | 390 | 400 | 410 | 420 |
| FVFVPGPEDP | GFGSILPRPP | LAESITQEFR | QRVPFSVFTT | NPCRIQYCTQ | EIIIFREDLV |
| 430 | 440 | 450 | 460 | 470 | 480 |
| NKMCRNCVRF | PSSSLDIPTH | FVKTILSQGH | LAPLPLYVCP | VHWAYDYTLR | VYPVPDLLVI |
| 490 | 500 | 510 | 520 | ||
| ADKYDPFTVT | NTDCLCINPG | SFPRSGFAFK | VFYPSSKTVE | DSKLQGF |