O13705
Gene name |
sec10 (SPAC13F5.06c) |
Protein name |
Exocyst complex component sec10 |
Names |
|
Species |
Schizosaccharomyces pombe (strain 972 / ATCC 24843) (Fission yeast) |
KEGG Pathway |
spo:SPAC13F5.06c |
EC number |
|
Protein Class |
|
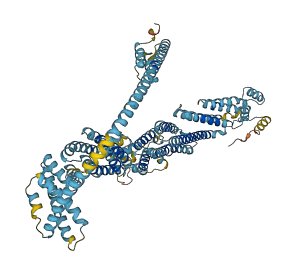
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for O13705
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-O13705-F1 | Predicted | AlphaFoldDB |
17 variants for O13705
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| I_2183937_G_C | 55 | I>M | No | Jeffares_SNPs | |
| I_2183507_C_A | 199 | A>S | No | Jeffares_SNPs | |
| I_2183377_G_A | 242 | A>V | No | Jeffares_SNPs | |
| I_2183067_C_G | 345 | K>N | No | Jeffares_SNPs | |
| I_2182631_T_A | 491 | I>F | No | Jeffares_SNPs | |
| I_2182614_G_T | 496 | N>K | No | Jeffares_SNPs | |
| I_2182613_G_A | 497 | H>Y | No | Jeffares_SNPs | |
| I_2182607_G_A | 499 | H>Y | No | Jeffares_SNPs | |
| I_2182599_A_C | 501 | N>K | No | Jeffares_SNPs | |
| I_2182456_A_C | 549 | F>C | No | Jeffares_SNPs | |
| I_2182412_T_C | 564 | K>E | No | Jeffares_SNPs | |
| I_2182379_C_T | 575 | D>N | No | Jeffares_SNPs | |
| I_2182223_A_G | 627 | F>L | No | Jeffares_SNPs | |
| I_2182213_G_A | 630 | T>I | No | Jeffares_SNPs | |
| I_2182066_T_C | 679 | K>R | No | Jeffares_SNPs | |
| I_2181985_A_C | 706 | M>R | No | Jeffares_SNPs | |
| I_2181611_G_A | 798 | Q>* | No | Jeffares_SNPs |
No associated diseases with O13705
No regional properties for O13705
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| No domain, repeats, and functional sites for O13705 | |||
5 GO annotations of cellular component
| Name | Definition |
|---|---|
| cell division site | The eventual plane of cell division (also known as cell cleavage or cytokinesis) in a dividing cell. In Eukaryotes, the cleavage apparatus, composed of septin structures and the actomyosin contractile ring, forms along this plane, and the mitotic, or meiotic, spindle is aligned perpendicular to the division plane. In bacteria, the cell division site is generally located at mid-cell and is the site at which the cytoskeletal structure, the Z-ring, assembles. |
| cell tip | The region at the end of the longest axis of a cylindrical or elongated cell. |
| cytosol | The part of the cytoplasm that does not contain organelles but which does contain other particulate matter, such as protein complexes. |
| exocyst | A protein complex peripherally associated with the plasma membrane that determines where vesicles dock and fuse. At least eight complex components are conserved between yeast and mammals. |
| nucleus | A membrane-bounded organelle of eukaryotic cells in which chromosomes are housed and replicated. In most cells, the nucleus contains all of the cell's chromosomes except the organellar chromosomes, and is the site of RNA synthesis and processing. In some species, or in specialized cell types, RNA metabolism or DNA replication may be absent. |
No GO annotations of molecular function
| Name | Definition |
|---|---|
| No GO annotations for molecular function |
4 GO annotations of biological process
| Name | Definition |
|---|---|
| exocytosis | A process of secretion by a cell that results in the release of intracellular molecules (e.g. hormones, matrix proteins) contained within a membrane-bounded vesicle. Exocytosis can occur either by full fusion, when the vesicle collapses into the plasma membrane, or by a kiss-and-run mechanism that involves the formation of a transient contact, a pore, between a granule (for exemple of chromaffin cells) and the plasma membrane. The latter process most of the time leads to only partial secretion of the granule content. Exocytosis begins with steps that prepare vesicles for fusion with the membrane (tethering and docking) and ends when molecules are secreted from the cell. |
| Golgi to plasma membrane transport | The directed movement of substances from the Golgi to the plasma membrane in transport vesicles that move from the trans-Golgi network to the plasma membrane, where they fuse and release their contents by exocytosis. |
| intracellular protein transport | The directed movement of proteins in a cell, including the movement of proteins between specific compartments or structures within a cell, such as organelles of a eukaryotic cell. |
| vesicle tethering involved in exocytosis | The initial, indirect interaction between a secretory vesicle membrane and a site of exocytosis in the plasma membrane. This interaction is mediated by tethering factors (or complexes), which interact with both membranes. Interaction can occur via direct binding to membrane phospholipids or membrane proteins, or via binding to vesicle coat proteins. This process is distinct from and prior to docking and fusion. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MSTKNALNDS | QIKLLNSLND | NKGIPSTEFV | EKFAESLYET | QNDGSKKLSS | IDGSIKSFAA |
| 70 | 80 | 90 | 100 | 110 | 120 |
| CLHELNRLKS | RVGDRIRDYA | SASKQVQNEY | HQKSNHLREK | FAQVLELSRH | LEDNVNDMRS |
| 130 | 140 | 150 | 160 | 170 | 180 |
| GLVDAGQELE | RAENNRKRIL | SSAELLRYYL | EFRSGKPQTL | MDFFRTNNHD | KMLLCAQRTR |
| 190 | 200 | 210 | 220 | 230 | 240 |
| QLLALANEVD | LPDSSETLAR | IEKFSEFLET | NFLKFFNNEY | RKPNWKGMAS | FGTILQEFNG |
| 250 | 260 | 270 | 280 | 290 | 300 |
| GASVVREFVN | QHEFFIAADK | VQSRQGLEQD | PIWLILPDPT | QKIPPLIQTL | SSLFSELCSV |
| 310 | 320 | 330 | 340 | 350 | 360 |
| IEGDCAVIKR | VFPNPELVLQ | TFFQRIFGQS | IQNRLEEVME | IAKGKSNLAY | LRTLQTVVSS |
| 370 | 380 | 390 | 400 | 410 | 420 |
| LRKLVADLKT | ILENRGFSVS | DNSPLSLALN | QYMEDLLVPF | IEVDDYLKRE | EHSLRSLFRL |
| 430 | 440 | 450 | 460 | 470 | 480 |
| SLYKYTSYKI | RLETPEPGLL | RSLMTPLQGN | MVAPTGVHSQ | FNTKTEGFLL | RIADIQENLI |
| 490 | 500 | 510 | 520 | 530 | 540 |
| QSGSFITEDY | ITIEKNHSHL | NSEKVYSFIG | WHAEALNRAS | ILISSQDLSV | VISSLVNLLD |
| 550 | 560 | 570 | 580 | 590 | 600 |
| KLIREDYVFK | ELSSIQSYIS | SHDKSKNLDL | HYLVDIRECK | KIMGYFSAYL | MSIVIPFTGV |
| 610 | 620 | 630 | 640 | 650 | 660 |
| TASSRRETVN | ILSSSISVIE | CAVNDVFYAT | VHALGDHLEI | ILSPYRQISY | AMTEEQIDSS |
| 670 | 680 | 690 | 700 | 710 | 720 |
| TELRQSMTRN | VQNYLDYIKN | LYHRLGPYDP | SLLALKQKTA | TMLAAMLISF | AFRSKVTAAG |
| 730 | 740 | 750 | 760 | 770 | 780 |
| ALLLQNDINF | FHSTLTSWGI | DTVDAKFKLI | LQLLSLLMVK | IDVLPAVMQD | KRKAGFSEMN |
| 790 | 800 | 810 | |||
| IHEVLRLRFD | LPENLKLQLN | KEEALLPPKS | S |