C1CES2
Gene name |
atpA |
Protein name |
V-type ATP synthase alpha chain |
Names |
V-ATPase subunit A |
Species |
Streptococcus pneumoniae (strain JJA) |
KEGG Pathway |
sjj:SPJ_1233 |
EC number |
7.1.2.2: Hydron translocation linked to the hydrolysis of a nucleoside triphosphate |
Protein Class |
|
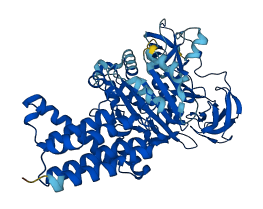
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for C1CES2
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-C1CES2-F1 | Predicted | AlphaFoldDB |
No variants for C1CES2
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for C1CES2 | |||||
No associated diseases with C1CES2
4 regional properties for C1CES2
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | ATPase, F1/V1/A1 complex, alpha/beta subunit, nucleotide-binding domain | 213 - 436 | IPR000194 |
| domain | ATPase, F1/V1/A1 complex, alpha/beta subunit, N-terminal domain | 6 - 68 | IPR004100 |
| active_site | ATPase, alpha/beta subunit, nucleotide-binding domain, active site | 427 - 436 | IPR020003 |
| domain | ATPsynthase alpha/beta subunit, N-terminal extension | 84 - 204 | IPR031686 |
Functions
| Description | ||
|---|---|---|
| EC Number | 7.1.2.2 | Hydron translocation linked to the hydrolysis of a nucleoside triphosphate |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
1 GO annotations of cellular component
| Name | Definition |
|---|---|
| proton-transporting ATP synthase complex | A proton-transporting two-sector ATPase complex that catalyzes the phosphorylation of ADP to ATP during oxidative phosphorylation. The complex comprises a membrane sector (F0) that carries out proton transport and a cytoplasmic compartment sector (F1) that catalyzes ATP synthesis by a rotational mechanism; the extramembrane sector (containing 3 a and 3 b subunits) is connected via the d-subunit to the membrane sector by several smaller subunits. Within this complex, the g and e subunits and the 9-12 c subunits rotate by consecutive 120 degree angles and perform parts of ATP synthesis. This movement is driven by the hydrogen ion electrochemical potential gradient. |
3 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| proton-transporting ATP synthase activity, rotational mechanism | Enables the synthesis of ATP from ADP and phosphate by the transfer of protons from one side of a membrane to the other by a rotational mechanism driven by a gradient according to the reaction: ADP + H2O + phosphate + H+(in) -> ATP + H+(out). |
| proton-transporting ATPase activity, rotational mechanism | Enables the transfer of protons from one side of a membrane to the other according to the reaction: ATP + H2O + H+(in) = ADP + phosphate + H+(out), by a rotational mechanism. |
1 GO annotations of biological process
| Name | Definition |
|---|---|
| proton motive force-driven plasma membrane ATP synthesis | The transport of protons across the plasma membrane to generate an electrochemical gradient (proton-motive force) that powers ATP synthesis. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MTQGKIIKVS | GPLVIASGMQ | EANIQDICRV | GKLGLIGEII | EMRRDQASIQ | VYEETSGLGP |
| 70 | 80 | 90 | 100 | 110 | 120 |
| GEPVVTTGEP | LSVELGPGLI | SQMFDGIQRP | LDRFKLATHN | DFLVRGVEVP | SLDRDIKWHF |
| 130 | 140 | 150 | 160 | 170 | 180 |
| DSTIAIGQKV | STGDILGTVK | ETEVVNHKIM | VPYGVSGEVV | SIASGDFTID | EVVYEIKKLD |
| 190 | 200 | 210 | 220 | 230 | 240 |
| GSFYKGTLMQ | KWPVRKARPV | SKRLIPEEPL | ITGQRVIDAF | FPVTKGGAAA | VPGPFGAGKT |
| 250 | 260 | 270 | 280 | 290 | 300 |
| VVQHQVAKFA | NVDIVIYVGC | GERGNEMTDV | LNEFPELIDP | NTGQSIMQRT | VLIANTSNMP |
| 310 | 320 | 330 | 340 | 350 | 360 |
| VAAREASIYT | GITMAEYFRD | MGYSVAIMAD | STSRWAEALR | EMSGRLEEMP | GDEGYPAYLG |
| 370 | 380 | 390 | 400 | 410 | 420 |
| SRIAEYYERA | GRSQVLGLPE | REGTITAIGA | VSPPGGDISE | PVTQNTLRIV | KVFWGLDAPL |
| 430 | 440 | 450 | 460 | 470 | 480 |
| AQRRHFPAIN | WLTSYSLYKD | SVGTYIDGKE | KTDWNSKITR | AMNYLQRESS | LEEIVRLVGI |
| 490 | 500 | 510 | 520 | 530 | 540 |
| DSLSDNERLT | MEIAKQIRED | YLQQNAFDSV | DTFTSFAKQE | AMLSNILTFA | DQANHALELG |
| 550 | 560 | 570 | 580 | 590 | |
| SYFTEIMEGT | VAVRDRMARS | KYVSEDRLDE | IKIISNEITH | QIHLILETGG | L |