B7J127
Gene name |
atpA |
Protein name |
V-type ATP synthase alpha chain |
Names |
V-ATPase subunit A |
Species |
Borreliella burgdorferi (strain ZS7) (Borrelia burgdorferi) |
KEGG Pathway |
bbz:BbuZS7_0094 |
EC number |
7.1.2.2: Hydron translocation linked to the hydrolysis of a nucleoside triphosphate |
Protein Class |
|
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
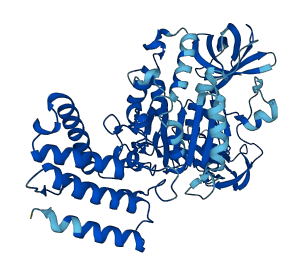
1 structures for B7J127
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-B7J127-F1 | Predicted | AlphaFoldDB |
No variants for B7J127
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for B7J127 | |||||
No associated diseases with B7J127
3 regional properties for B7J127
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | ATPase, F1/V1/A1 complex, alpha/beta subunit, nucleotide-binding domain | 220 - 439 | IPR000194 |
| domain | ATPase, F1/V1/A1 complex, alpha/beta subunit, N-terminal domain | 7 - 70 | IPR004100 |
| domain | ATPsynthase alpha/beta subunit, N-terminal extension | 87 - 209 | IPR031686 |
Functions
| Description | ||
|---|---|---|
| EC Number | 7.1.2.2 | Hydron translocation linked to the hydrolysis of a nucleoside triphosphate |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
1 GO annotations of cellular component
| Name | Definition |
|---|---|
| proton-transporting ATP synthase complex | A proton-transporting two-sector ATPase complex that catalyzes the phosphorylation of ADP to ATP during oxidative phosphorylation. The complex comprises a membrane sector (F0) that carries out proton transport and a cytoplasmic compartment sector (F1) that catalyzes ATP synthesis by a rotational mechanism; the extramembrane sector (containing 3 a and 3 b subunits) is connected via the d-subunit to the membrane sector by several smaller subunits. Within this complex, the g and e subunits and the 9-12 c subunits rotate by consecutive 120 degree angles and perform parts of ATP synthesis. This movement is driven by the hydrogen ion electrochemical potential gradient. |
3 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| proton-transporting ATP synthase activity, rotational mechanism | Enables the synthesis of ATP from ADP and phosphate by the transfer of protons from one side of a membrane to the other by a rotational mechanism driven by a gradient according to the reaction: ADP + H2O + phosphate + H+(in) -> ATP + H+(out). |
| proton-transporting ATPase activity, rotational mechanism | Enables the transfer of protons from one side of a membrane to the other according to the reaction: ATP + H2O + H+(in) = ADP + phosphate + H+(out), by a rotational mechanism. |
1 GO annotations of biological process
| Name | Definition |
|---|---|
| proton motive force-driven plasma membrane ATP synthesis | The transport of protons across the plasma membrane to generate an electrochemical gradient (proton-motive force) that powers ATP synthesis. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MNTKGKVVGV | NGNLVTIEVE | GSVFMNEVLF | VKTAGRNLKA | EVIRIRGNEV | DAQVFELTKG |
| 70 | 80 | 90 | 100 | 110 | 120 |
| ISVGDLVEFT | DKLLTVELGP | GLLTQVYDGL | QNPLPELAIQ | CGFFLERGVY | LRPLNKDKKW |
| 130 | 140 | 150 | 160 | 170 | 180 |
| NFKKTSKVGD | IVIAGDFLGF | VIEGTVHHQI | MIPFYKRDSY | KIVEIVSDGD | YSIDEQIAVI |
| 190 | 200 | 210 | 220 | 230 | 240 |
| EDDSGMRHNI | TMSFHWPVKV | PITNYKERLI | PSEPMLTQTR | IIDTFFPVAK | GGTFCIPGPF |
| 250 | 260 | 270 | 280 | 290 | 300 |
| GAGKTVLQQV | TSRNADVDVV | IIAACGERAG | EVVETLKEFP | ELMDPKTGKS | LMDRTCIICN |
| 310 | 320 | 330 | 340 | 350 | 360 |
| TSSMPVAARE | ASVYTAITIG | EYYRQMGLDI | LLLADSTSRW | AQAMREMSGR | LEEIPGEEAF |
| 370 | 380 | 390 | 400 | 410 | 420 |
| PAYLESVIAS | FYERAGIVVL | NNGDIGSVTV | GGSVSPAGGN | FEEPVTQATL | KVVGAFHGLT |
| 430 | 440 | 450 | 460 | 470 | 480 |
| RERSDARKFP | AISPLESWSK | YKGVIDQKKT | EYARSFLVKG | NEINQMMKVV | GEEGISNDDF |
| 490 | 500 | 510 | 520 | 530 | 540 |
| LIYLKSELLD | SCYLQQNSFD | SIDAAVSSER | QNYMFDIVYN | ILKTNFEFSD | KLQARDFINE |
| 550 | 560 | 570 | |||
| LRQNLLDMNL | SSFKDHKFNK | LEHALGELIN | FKKVI |