B2G6L2
Gene name |
ileS |
Protein name |
Isoleucine--tRNA ligase |
Names |
Isoleucyl-tRNA synthetase, IleRS |
Species |
Limosilactobacillus reuteri (strain JCM 1112) (Lactobacillus reuteri) |
KEGG Pathway |
lrf:LAR_0578 |
EC number |
6.1.1.5: Ligases forming aminoacyl-tRNA and related compounds |
Protein Class |
|
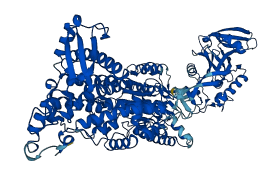
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for B2G6L2
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-B2G6L2-F1 | Predicted | AlphaFoldDB |
No variants for B2G6L2
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for B2G6L2 | |||||
No associated diseases with B2G6L2
5 regional properties for B2G6L2
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| conserved_site | Aminoacyl-tRNA synthetase, class I, conserved site | 57 - 68 | IPR001412 |
| domain | Aminoacyl-tRNA synthetase, class Ia | 29 - 635 | IPR002300 |
| domain | Zinc finger, FPG/IleRS-type | 887 - 915 | IPR010663 |
| domain | Methionyl/Valyl/Leucyl/Isoleucyl-tRNA synthetase, anticodon-binding | 679 - 831 | IPR013155 |
| domain | Isoleucyl tRNA synthetase type 1, anticodon-binding domain | 634 - 811 | IPR033708 |
Functions
| Description | ||
|---|---|---|
| EC Number | 6.1.1.5 | Ligases forming aminoacyl-tRNA and related compounds |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
1 GO annotations of cellular component
| Name | Definition |
|---|---|
| cytoplasm | The contents of a cell excluding the plasma membrane and nucleus, but including other subcellular structures. |
5 GO annotations of molecular function
| Name | Definition |
|---|---|
| aminoacyl-tRNA editing activity | The hydrolysis of an incorrectly aminoacylated tRNA. |
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| isoleucine-tRNA ligase activity | Catalysis of the reaction: L-isoleucine + ATP + tRNA(Ile) = L-isoleucyl-tRNA(Ile) + AMP + diphosphate + 2 H(+). |
| tRNA binding | Binding to a transfer RNA. |
| zinc ion binding | Binding to a zinc ion (Zn). |
1 GO annotations of biological process
| Name | Definition |
|---|---|
| isoleucyl-tRNA aminoacylation | The process of coupling isoleucine to isoleucyl-tRNA, catalyzed by isoleucyl-tRNA synthetase. The isoleucyl-tRNA synthetase is a class-I synthetase. The activated amino acid is transferred to the 2'-OH group of a isoleucine-accetping tRNA. The 2'-O-aminoacyl-tRNA will ultimately migrate to the 3' position via transesterification. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MRVKDTLNLG | RTKFPMRGKL | PVTEAQREQL | WEENKVYELR | QKLNEGKPTF | VLHDGPPYAN |
| 70 | 80 | 90 | 100 | 110 | 120 |
| GNIHIGHAMN | KISKDFIVRY | KSMSGYRAPY | VPGWDTHGLP | IEHQLTKSGY | DRKKMSLTEF |
| 130 | 140 | 150 | 160 | 170 | 180 |
| RDLCREYALK | QVDKQRTDFK | RLGVSGEWDH | PYLTLDKEFE | AAQIRVFGEF | AKKGLLYQAK |
| 190 | 200 | 210 | 220 | 230 | 240 |
| KPVYWSWSSE | SALAEAEVEY | HDVVAKTAFF | VEQIKDGKGR | LDNDTYLVVW | TTTPWTVPAS |
| 250 | 260 | 270 | 280 | 290 | 300 |
| EAVAVNPKFD | YSVVNPANDD | RKFVVATDLL | EKLAEKLGWE | DYEVVDHLMG | QELEGMTTQH |
| 310 | 320 | 330 | 340 | 350 | 360 |
| PYLDRDLLVG | LADYVTADAG | TGLVHTAPGY | GDDDYNFGKK | YDLPIFAPIN | DQGVLTKENG |
| 370 | 380 | 390 | 400 | 410 | 420 |
| EGFEGVFYQD | ADDVSLQKLE | ENNALLLQEP | LQHSYPFDWR | TKQPIIFRAT | DQWFVSIEKM |
| 430 | 440 | 450 | 460 | 470 | 480 |
| RQNILDALED | VKYHPEWGKV | RLRNMIKDRG | DWVISRQRVW | GVPLPIFYAE | DGTPIMEEET |
| 490 | 500 | 510 | 520 | 530 | 540 |
| INHVAELFAK | YGSNVWFERE | AKDLLPEGYT | NEHSPNGKFT | KETDIMDVWF | DSGSSHQGVL |
| 550 | 560 | 570 | 580 | 590 | 600 |
| AERDYLTYPA | DLYLEGSDQY | RGWFNSSLIT | SVVCSGHAPY | KEIVSQGFTL | DKRGNKMSKS |
| 610 | 620 | 630 | 640 | 650 | 660 |
| QGNVIDPNKV | VQQMGAEIIR | LWVMSADTSA | DVRVSMGTFQ | QISEAYRKLR | NTFRFLLANT |
| 670 | 680 | 690 | 700 | 710 | 720 |
| SDFNPEENTV | SYEKLQSVDK | YMLVKLNHFL | KTMREDFDNY | DFLDAYKVLI | NFVNNDLSAF |
| 730 | 740 | 750 | 760 | 770 | 780 |
| YMNIAKDVLY | IEAENSEVRR | SMQTVFYDIL | LTLVKLLTPI | LPHTTEEVWS | YMNEPEDFVQ |
| 790 | 800 | 810 | 820 | 830 | 840 |
| LTEIPDPRTF | AGEEELLSKW | DDFMEVRSHV | LKSLEEARNA | KLIGKSLEAQ | VDLYLTDDQK |
| 850 | 860 | 870 | 880 | 890 | 900 |
| QLLDSLNENI | QLLLGVSALH | VHPADEAPAD | ADQYNDGVAV | KVTTANGETC | ARCRMVKEDV |
| 910 | 920 | 930 | |||
| GSDPAYPELC | ARCAAIVREN | FPETAEDGLE | E |