A9FDV9
Gene name |
ftsH2 |
Protein name |
ATP-dependent zinc metalloprotease FtsH 2 |
Names |
|
Species |
Sorangium cellulosum (strain So ce56) (Polyangium cellulosum (strain So ce56)) |
KEGG Pathway |
scl:sce1641 |
EC number |
|
Protein Class |
|
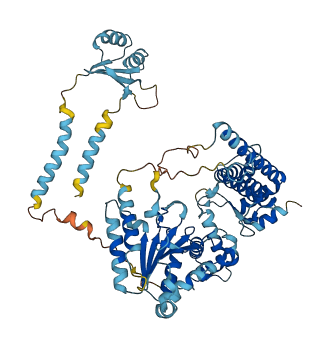
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for A9FDV9
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-A9FDV9-F1 | Predicted | AlphaFoldDB |
No variants for A9FDV9
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for A9FDV9 | |||||
No associated diseases with A9FDV9
9 regional properties for A9FDV9
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | Elongation factor EFG, domain V-like | 609 - 697 | IPR000640 |
| domain | Translational (tr)-type GTP-binding domain | 8 - 290 | IPR000795 |
| domain | Translation elongation factor EFTu-like, domain 2 | 331 - 398 | IPR004161 |
| domain | Small GTP-binding protein domain | 10 - 186 | IPR005225 |
| domain | Translation elongation factor EFG/EF2, domain IV | 486 - 607 | IPR005517 |
| domain | Elongation factor G, domain III | 412 - 487 | IPR009022 |
| conserved_site | Tr-type G domain, conserved site | 51 - 66 | IPR031157 |
| domain | EFG, domain V | 612 - 690 | IPR035649 |
| domain | Elongation Factor G, domain II | 411 - 484 | IPR041095 |
2 GO annotations of cellular component
| Name | Definition |
|---|---|
| integral component of membrane | The component of a membrane consisting of the gene products and protein complexes having at least some part of their peptide sequence embedded in the hydrophobic region of the membrane. |
| plasma membrane | The membrane surrounding a cell that separates the cell from its external environment. It consists of a phospholipid bilayer and associated proteins. |
5 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| ATP hydrolysis activity | Catalysis of the reaction: ATP + H2O = ADP + H+ phosphate. ATP hydrolysis is used in some reactions as an energy source, for example to catalyze a reaction or drive transport against a concentration gradient. |
| ATP-dependent peptidase activity | Catalysis of the hydrolysis of peptide bonds, driven by ATP hydrolysis. |
| metalloendopeptidase activity | Catalysis of the hydrolysis of internal, alpha-peptide bonds in a polypeptide chain by a mechanism in which water acts as a nucleophile, one or two metal ions hold the water molecule in place, and charged amino acid side chains are ligands for the metal ions. |
| zinc ion binding | Binding to a zinc ion (Zn). |
2 GO annotations of biological process
| Name | Definition |
|---|---|
| protein catabolic process | The chemical reactions and pathways resulting in the breakdown of a protein by the destruction of the native, active configuration, with or without the hydrolysis of peptide bonds. |
| proteolysis | The hydrolysis of proteins into smaller polypeptides and/or amino acids by cleavage of their peptide bonds. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MRSLWIVLVL | VLGSALLLQV | MAASDDRIPY | ARFRSLAERG | ELAEIEIRDD | MYIGRAVSGL |
| 70 | 80 | 90 | 100 | 110 | 120 |
| SARAPQSYRT | GRIEQTEKDL | LADLDRRGIP | YTRVADELGL | PPYLWLLLPL | AGLAAMGHLA |
| 130 | 140 | 150 | 160 | 170 | 180 |
| SRRATTAGTI | SGAATAFGKH | KARLYEERGA | IATFRDVAGN | AEAKTELSEI | VDFLKAPERY |
| 190 | 200 | 210 | 220 | 230 | 240 |
| EKLGGRMPRG | VLLVGPPGTG | KTLLARAIAG | EASVPFFSAS | GSEFVEMFVG | VGAARVRDLF |
| 250 | 260 | 270 | 280 | 290 | 300 |
| SQAREKGACL | VFIDELDAVG | KVRGLGGSVG | GHDEREQTLN | QLLTEMDGFD | AHTAMVVIGA |
| 310 | 320 | 330 | 340 | 350 | 360 |
| TNRAEILDPA | LLRPGRFDRR | VHIDRPDLAE | RKEILAVHAR | KVALDPGADL | DAVAAQTAGL |
| 370 | 380 | 390 | 400 | 410 | 420 |
| VGADLANIVN | EAALLAARRG | AEAVGHGDLE | AAIERGLAGL | ERRGRRLGAR | EKLVVAYHEV |
| 430 | 440 | 450 | 460 | 470 | 480 |
| GHALTASLLP | TQDPVRKVSI | VPRGPGALGY | TIQQPREDRY | LWSRQEILDR | LVVLLGGRVA |
| 490 | 500 | 510 | 520 | 530 | 540 |
| EEEAVGDLST | GAQDDLLNAT | ELARRMVREL | GMGQGLGLSA | LEPRRPLSFL | GEAQGAMPSG |
| 550 | 560 | 570 | 580 | 590 | 600 |
| AGPRECSDAT | ARAIDAEVAR | ILADAEARAR | ALIQGHRPTL | ERVAARLYEV | ETLSGDELRE |
| MVASGEA |