A8X6H1
Gene name |
egl-4 |
Protein name |
cGMP-dependent protein kinase egl-4 |
Names |
Egg-laying defective protein 4 |
Species |
Caenorhabditis briggsae |
KEGG Pathway |
|
EC number |
2.7.11.12: Protein-serine/threonine kinases |
Protein Class |
|
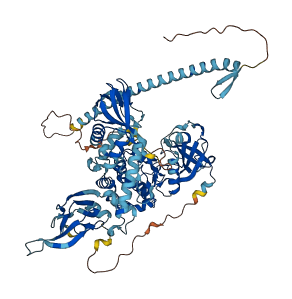
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
579-601 (Activation loop from InterPro)
Target domain |
438-698 (Protein kinase domain) |
Relief mechanism |
|
Assay |
|
Autoinhibited structure

Activated structure
1 structures for A8X6H1
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-A8X6H1-F1 | Predicted | AlphaFoldDB |
No variants for A8X6H1
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for A8X6H1 | |||||
No associated diseases with A8X6H1
4 regional properties for A8X6H1
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | Translation elongation factor P/YeiP, central | 68 - 128 | IPR001059 |
| domain | Translation elongation factor, KOW-like | 4 - 61 | IPR013185 |
| conserved_site | Translation elongation factor P/YeiP, conserved site | 152 - 171 | IPR013852 |
| domain | Elongation factor P, C-terminal | 131 - 186 | IPR015365 |
Functions
| Description | ||
|---|---|---|
| EC Number | 2.7.11.12 | Protein-serine/threonine kinases |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
2 GO annotations of cellular component
| Name | Definition |
|---|---|
| cytoplasm | The contents of a cell excluding the plasma membrane and nucleus, but including other subcellular structures. |
| nucleus | A membrane-bounded organelle of eukaryotic cells in which chromosomes are housed and replicated. In most cells, the nucleus contains all of the cell's chromosomes except the organellar chromosomes, and is the site of RNA synthesis and processing. In some species, or in specialized cell types, RNA metabolism or DNA replication may be absent. |
5 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| cGMP binding | Binding to cGMP, the nucleotide cyclic GMP (guanosine 3',5'-cyclophosphate). |
| cGMP-dependent protein kinase activity | cGMP dependent catalysis of the reaction: ATP + a protein = ADP + a phosphoprotein. |
| metal ion binding | Binding to a metal ion. |
| protein serine kinase activity | Catalysis of the reactions: ATP + protein serine = ADP + protein serine phosphate. |
2 GO annotations of biological process
| Name | Definition |
|---|---|
| chemotaxis | The directed movement of a motile cell or organism, or the directed growth of a cell guided by a specific chemical concentration gradient. Movement may be towards a higher concentration (positive chemotaxis) or towards a lower concentration (negative chemotaxis). |
| protein phosphorylation | The process of introducing a phosphate group on to a protein. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MYGSSRHHLD | SFSSNDGNAF | LVQVGSRTFE | AHELQKLIPQ | LEEAISRKDA | QLRQQQSIVE |
| 70 | 80 | 90 | 100 | 110 | 120 |
| GHIKRISELE | GEVTTLQREC | DKLRSVLEQK | AQSAASPGQP | PSPSPRTDQL | GNDLQQKAVF |
| 130 | 140 | 150 | 160 | 170 | 180 |
| PADGTQQRAK | KIAVSAEPTN | FENKPATLQH | YNKTVAAKQM | IRDAVQKNDF | LKQLAKEQII |
| 190 | 200 | 210 | 220 | 230 | 240 |
| ELVNCMYEMR | ARAGQWVIQE | GEPGDRLFVV | AEGELQVSRE | GATLGKMRAG | TVMGELAILY |
| 250 | 260 | 270 | 280 | 290 | 300 |
| NCTRTASVQA | LTDVQLWVLD | RSVFQMITQR | LGMERHSQII | NFLSKVSIFA | NLTEDRISKI |
| 310 | 320 | 330 | 340 | 350 | 360 |
| ADVMDQDYYD | GGHYILRQGE | KGDAFFVINS | GQVKVTQQIE | GEKEAREIRI | LNQGDFFGER |
| 370 | 380 | 390 | 400 | 410 | 420 |
| ALLGDEVRTA | NIIAQAPGVE | VLTLDRESFT | KLIGDLDTLR | KDYGDKERVA | TLVREPPSPV |
| 430 | 440 | 450 | 460 | 470 | 480 |
| KIVDDFREEF | ANVTLKNVKR | LATLGVGGFG | RVELVCVNGD | KSKTYALKAL | KKKHIVDTRQ |
| 490 | 500 | 510 | 520 | 530 | 540 |
| QEHIFAERNI | MMETSTDWIV | KLYKTFRDQK | FVYMLLEVCL | GGELWTTLRD | RGHFDDYTAR |
| 550 | 560 | 570 | 580 | 590 | 600 |
| FYVACVLEGL | EYLHRKNIVY | RDLKPENCLL | ANSGYLKLVD | FGFAKKLASG | RKTWTFCGTP |
| 610 | 620 | 630 | 640 | 650 | 660 |
| EYVSPEIILN | KGHDQAADYW | ALGIYICELM | LGRPPFQASD | PMKTYTLILK | GVDALEIPNR |
| 670 | 680 | 690 | 700 | 710 | 720 |
| RIGKTATALV | KKLCRDNPGE | RLGSGSGGVN | DIRKHRWFMG | FDWEGLRTKT | LKPPILPKVN |
| 730 | 740 | ||||
| NPADVTNFDN | YPPDNDVPPD | EFSGWDEGF |