A8IA58
Gene name |
phnN (AZC_2467) |
Protein name |
Bifunctional ribose 1,5-bisphosphokinase-thymidine phosphorylase |
Names |
|
Species |
Azorhizobium caulinodans (strain ATCC 43989 / DSM 5975 / JCM 20966 / LMG 6465 / NBRC 14845 / NCIMB 13405 / ORS 571) |
KEGG Pathway |
azc:AZC_2467 |
EC number |
2.4.2.4: Pentosyltransferases |
Protein Class |
|
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
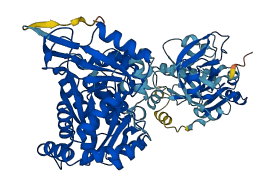
1 structures for A8IA58
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-A8IA58-F1 | Predicted | AlphaFoldDB |
No variants for A8IA58
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for A8IA58 | |||||
No associated diseases with A8IA58
4 regional properties for A8IA58
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | Glycosyl transferase, family 3 | 349 - 489 | IPR000312 |
| domain | Guanylate kinase/L-type calcium channel beta subunit | 6 - 186 | IPR008145 |
| domain | Pyrimidine nucleoside phosphorylase, C-terminal | 611 - 678 | IPR013102 |
| conserved_site | Pyrimidine-nucleoside phosphorylase, conserved site | 383 - 398 | IPR017872 |
Functions
| Description | ||
|---|---|---|
| EC Number | 2.4.2.4 | Pentosyltransferases |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
No GO annotations of cellular component
| Name | Definition |
|---|---|
| No GO annotations for cellular component |
4 GO annotations of molecular function
| Name | Definition |
|---|---|
| 1,4-alpha-oligoglucan phosphorylase activity | Catalysis of the reaction: 1,4-alpha-D-glucosyl(n) + phosphate = 1,4-alpha-D-glucosyl(n-1) + alpha-D-glucose 1-phosphate. The name should be qualified in each instance by adding the name of the natural substrate, e.g. maltodextrin phosphorylase, starch phosphorylase, glycogen phosphorylase. |
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| ribose 1,5-bisphosphate phosphokinase activity | Catalysis of the reaction: D-ribose 1,5-diphosphate + ATP = 5-phospho-alpha-D-ribose 1-diphosphate + ADP + H(+). |
| thymidine phosphorylase activity | Catalysis of the reaction: thymidine + phosphate = thymine + 2-deoxy-D-ribose 1-phosphate. |
5 GO annotations of biological process
| Name | Definition |
|---|---|
| 5-phosphoribose 1-diphosphate biosynthetic process | The chemical reactions and pathways resulting in the formation of 5-phosphoribose 1-diphosphate, also known as 5-phosphoribosyl-1-pyrophosphate. |
| organic phosphonate metabolic process | The chemical reactions and pathways involving phosphonates, any organic compounds containing one or more C-PO(OH)2 or C-PO(OR)2 (with R=alkyl, aryl) groups. Metabolism of phosphonic acid itself, an inorganic compound without the biochemically relevant C-P bond, is not included. |
| organic phosphonate transport | The directed movement of phosphonates into, out of or within a cell, or between cells, by means of some agent such as a transporter or pore. A phosphonate is any salt, anion, or ester of phosphonic acid (HPO(OH)2). |
| pyrimidine nucleobase metabolic process | The chemical reactions and pathways involving pyrimidine nucleobases, 1,3-diazine, organic nitrogenous bases. |
| pyrimidine nucleoside metabolic process | The chemical reactions and pathways involving any pyrimidine nucleoside, one of a family of organic molecules consisting of a pyrimidine base covalently bonded to ribose (a ribonucleoside) or deoxyribose (a deoxyribonucleoside). |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MSVMGSGLFF | FVVGPSGSGK | DTLIEGAKAA | LGPTGRYVFA | RRAITRPADA | GGEAHEALSV |
| 70 | 80 | 90 | 100 | 110 | 120 |
| DQFDAVLAQG | GFLIHWEAHG | LKYGLRATLL | DDMAAGRHVI | ANGSRAMVAA | LAERVPHLVV |
| 130 | 140 | 150 | 160 | 170 | 180 |
| VEITAPEAVL | AERLKGRGRE | GAENIAARLE | RKVPPFPESV | TVIQVPNDST | PRAGIEKFVA |
| 190 | 200 | 210 | 220 | 230 | 240 |
| ALVAQTARLR | LVRMAIETGR | RNVAFLARGN | TVVAAPDYLG | PGRVDLIGEG | RSIRAEVALV |
| 250 | 260 | 270 | 280 | 290 | 300 |
| GDALLPSDAV | GLSSEAFGAL | GLPEGAELVL | TRTPVPESRA | ALRRKIQGAT | LDEGAYAQVV |
| 310 | 320 | 330 | 340 | 350 | 360 |
| GDIVEGRYPD | SEVAGFLVAA | DRSLSDDEVL | ALAKVRAKFA | SRITWDEPMV | VDKHSMGGIP |
| 370 | 380 | 390 | 400 | 410 | 420 |
| GSRITMIVVP | IVAAHGLAIP | KTSSRAITSA | AGTADAMETL | ARVDLDSAEV | RRTVERARGC |
| 430 | 440 | 450 | 460 | 470 | 480 |
| IAWNGRLSHS | ALDDVMNAIT | RPLGLDSTRW | SVASILSKKL | AAGSTHVVID | LPFGARARVK |
| 490 | 500 | 510 | 520 | 530 | 540 |
| GAGEAHEMAR | LFEQVGAGLG | LTVEAIPTDG | SAPIGRGIGP | ALEVRDVLWV | LEDHSEAPPD |
| 550 | 560 | 570 | 580 | 590 | 600 |
| LKEKALFFAS | RILAWDPAVG | PDRARARAEE | LLASGAARAA | LERIVEAQGR | WSEPVRPARL |
| 610 | 620 | 630 | 640 | 650 | 660 |
| THTVTAQNDG | QVSDIDGFAV | AGIARLAGAP | LDKGAGIDLK | ARVGDVVRAG | DPLFVIHAST |
| 670 | 680 | 690 | |||
| AADLEAAAGA | ALAFDGYGIM | MDGKAFRRIN | PER |