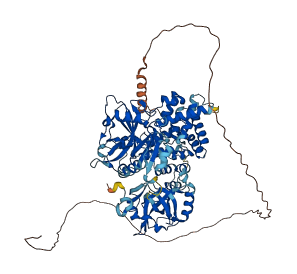
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for A6ZXG6
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-A6ZXG6-F1 | Predicted | AlphaFoldDB |
No variants for A6ZXG6
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for A6ZXG6 | |||||
No associated diseases with A6ZXG6
5 regional properties for A6ZXG6
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | DNA ligase, ATP-dependent, N-terminal | 147 - 323 | IPR012308 |
| domain | DNA ligase, ATP-dependent, C-terminal | 623 - 732 | IPR012309 |
| domain | DNA ligase, ATP-dependent, central | 393 - 636 | IPR012310 |
| conserved_site | DNA ligase, ATP-dependent, conserved site | 417 - 425 | IPR016059-1 |
| conserved_site | DNA ligase, ATP-dependent, conserved site | 571 - 598 | IPR016059-2 |
No GO annotations of cellular component
| Name | Definition |
|---|---|
| No GO annotations for cellular component |
3 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| DNA binding | Any molecular function by which a gene product interacts selectively and non-covalently with DNA (deoxyribonucleic acid). |
| DNA ligase (ATP) activity | Catalysis of the reaction: ATP + deoxyribonucleotide(n) + deoxyribonucleotide(m) = AMP + diphosphate + deoxyribonucleotide(n+m). |
4 GO annotations of biological process
| Name | Definition |
|---|---|
| DNA biosynthetic process | The biosynthetic process resulting in the formation of DNA. |
| DNA recombination | Any process in which a new genotype is formed by reassortment of genes resulting in gene combinations different from those that were present in the parents. In eukaryotes genetic recombination can occur by chromosome assortment, intrachromosomal recombination, or nonreciprocal interchromosomal recombination. Interchromosomal recombination occurs by crossing over. In bacteria it may occur by genetic transformation, conjugation, transduction, or F-duction. |
| DNA repair | The process of restoring DNA after damage. Genomes are subject to damage by chemical and physical agents in the environment (e.g. UV and ionizing radiations, chemical mutagens, fungal and bacterial toxins, etc.) and by free radicals or alkylating agents endogenously generated in metabolism. DNA is also damaged because of errors during its replication. A variety of different DNA repair pathways have been reported that include direct reversal, base excision repair, nucleotide excision repair, photoreactivation, bypass, double-strand break repair pathway, and mismatch repair pathway. |
| DNA replication | The cellular metabolic process in which a cell duplicates one or more molecules of DNA. DNA replication begins when specific sequences, known as origins of replication, are recognized and bound by initiation proteins, and ends when the original DNA molecule has been completely duplicated and the copies topologically separated. The unit of replication usually corresponds to the genome of the cell, an organelle, or a virus. The template for replication can either be an existing DNA molecule or RNA. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MRRLLTGCLL | SSARPLKSRL | PLLMSSSLPS | SAGKKPKQAT | LARFFTSMKN | KPTEGTPSPK |
| 70 | 80 | 90 | 100 | 110 | 120 |
| KSSKHMLEDR | MDNVSGEEEY | ATKKLKQTAV | THTVAAPSSM | GSNFSSIPSS | APSSGVADSP |
| 130 | 140 | 150 | 160 | 170 | 180 |
| QQSQRLVGEV | EDALSSNNND | HYSSNIPYSE | VCEVFNKIEA | ISSRLEIIRI | CSDFFIKIMK |
| 190 | 200 | 210 | 220 | 230 | 240 |
| QSSKNLIPTT | YLFINRLGPD | YEAGLELGLG | ENLLMKTISE | TCGKSMSQIK | LKYKDIGDLG |
| 250 | 260 | 270 | 280 | 290 | 300 |
| EIAMGARNVQ | PTMFKPKPLT | VGEVFKNLRA | IAKTQGKDSQ | LKKMKLIKRM | LTACKGIEAK |
| 310 | 320 | 330 | 340 | 350 | 360 |
| FLIRSLESKL | RIGLAEKTVL | ISLSKALLLH | DENREDSPDK | DVPMDVLESA | QQKIRDAFCQ |
| 370 | 380 | 390 | 400 | 410 | 420 |
| VPNYEIVINS | CLEHGIMNLD | KYCTLRPGIP | LKPMLAKPTK | AINEVLDRFQ | GETFTSEYKY |
| 430 | 440 | 450 | 460 | 470 | 480 |
| DGERAQVHLL | NDGTMRIYSR | NGENMTERYP | EINITDFIQD | LDTTKNLILD | CEAVAWDKDQ |
| 490 | 500 | 510 | 520 | 530 | 540 |
| GKILPFQVLS | TRKRKDVELN | DVKVKVCLFA | FDILCYNDER | LINKSLKERR | EYLTKVTKVV |
| 550 | 560 | 570 | 580 | 590 | 600 |
| PGEFQYATQI | TTNNLDELQK | FLDESVNHSC | EGLMVKMLEG | PESHYEPSKR | SRNWLKLKKD |
| 610 | 620 | 630 | 640 | 650 | 660 |
| YLEGVGDSLD | LCVLGAYYGR | GKRTGTYGGF | LLGCYNQDTG | EFETCCKIGT | GFSDEMLQLL |
| 670 | 680 | 690 | 700 | 710 | 720 |
| HDRLTPTIID | GPKATFVFDS | SAEPDVWFEP | TTLFEVLTAD | LSLSPIYKAG | SATFDKGVSL |
| 730 | 740 | 750 | |||
| RFPRFLRIRE | DKGVEDATSS | DQIVELYENQ | SHMQN |