A6QV55
Gene name |
FEN1 |
Protein name |
Flap endonuclease 1 |
Names |
FEN-1, Flap structure-specific endonuclease 1 |
Species |
Ajellomyces capsulatus (strain NAm1 / WU24) (Darling's disease fungus) (Histoplasma capsulatum) |
KEGG Pathway |
aje:HCAG_01262 |
EC number |
|
Protein Class |
|
Descriptions
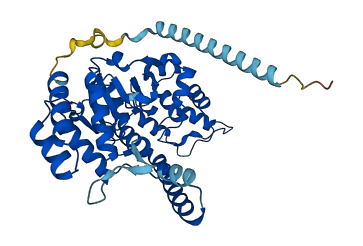
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for A6QV55
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-A6QV55-F1 | Predicted | AlphaFoldDB |
No variants for A6QV55
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for A6QV55 | |||||
No associated diseases with A6QV55
5 regional properties for A6QV55
| Type | Name | Position | InterPro Accession |
|---|---|---|---|
| domain | XPG, N-terminal | 1 - 107 | IPR006085 |
| domain | XPG-I domain | 146 - 233 | IPR006086 |
| conserved_site | Helix-hairpin-helix motif, class 2 | 220 - 253 | IPR008918 |
| conserved_site | XPG conserved site | 79 - 93 | IPR019974-1 |
| conserved_site | XPG conserved site | 149 - 163 | IPR019974-2 |
Functions
4 GO annotations of cellular component
| Name | Definition |
|---|---|
| cytosol | The part of the cytoplasm that does not contain organelles but which does contain other particulate matter, such as protein complexes. |
| mitochondrion | A semiautonomous, self replicating organelle that occurs in varying numbers, shapes, and sizes in the cytoplasm of virtually all eukaryotic cells. It is notably the site of tissue respiration. |
| nucleolus | A small, dense body one or more of which are present in the nucleus of eukaryotic cells. It is rich in RNA and protein, is not bounded by a limiting membrane, and is not seen during mitosis. Its prime function is the transcription of the nucleolar DNA into 45S ribosomal-precursor RNA, the processing of this RNA into 5.8S, 18S, and 28S components of ribosomal RNA, and the association of these components with 5S RNA and proteins synthesized outside the nucleolus. This association results in the formation of ribonucleoprotein precursors; these pass into the cytoplasm and mature into the 40S and 60S subunits of the ribosome. |
| nucleoplasm | That part of the nuclear content other than the chromosomes or the nucleolus. |
4 GO annotations of molecular function
| Name | Definition |
|---|---|
| 5'-3' exonuclease activity | Catalysis of the hydrolysis of ester linkages within nucleic acids by removing nucleotide residues from the 5' end. |
| 5'-flap endonuclease activity | Catalysis of the cleavage of a 5' flap structure in DNA, but not other DNA structures; processes the 5' ends of Okazaki fragments in lagging strand DNA synthesis. |
| DNA binding | Any molecular function by which a gene product interacts selectively and non-covalently with DNA (deoxyribonucleic acid). |
| magnesium ion binding | Binding to a magnesium (Mg) ion. |
5 GO annotations of biological process
| Name | Definition |
|---|---|
| base-excision repair | In base excision repair, an altered base is removed by a DNA glycosylase enzyme, followed by excision of the resulting sugar phosphate. The small gap left in the DNA helix is filled in by the sequential action of DNA polymerase and DNA ligase. |
| DNA replication, removal of RNA primer | Removal of the Okazaki RNA primer from the lagging strand of replicating DNA, by a combination of the actions of DNA polymerase, DNA helicase and an endonuclease. |
| double-strand break repair via nonhomologous end joining | The repair of a double-strand break in DNA in which the two broken ends are rejoined with little or no sequence complementarity. Information at the DNA ends may be lost due to the modification of broken DNA ends. This term covers instances of separate pathways, called classical (or canonical) and alternative nonhomologous end joining (C-NHEJ and A-NHEJ). These in turn may further branch into sub-pathways, but evidence is still unclear. |
| gene conversion at mating-type locus | The conversion of the mating-type locus from one allele to another resulting from the recombinational repair of a site-specific double-strand break at the mating-type locus with information from a silent donor sequence. There is no reciprocal exchange of information because the mating-type locus copies information from the donor sequence and the donor sequence remains unchanged. |
| maintenance of DNA trinucleotide repeats | Any process involved in sustaining the fidelity and copy number of DNA trinucleotide repeats. DNA trinucleotide repeats are naturally occurring runs of three base-pairs. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MGIKHLYQII | QENAPDAVKA | GEIKNHFGRK | VAIDASMSIY | SFLIAVRSDG | QQLTSETGET |
| 70 | 80 | 90 | 100 | 110 | 120 |
| TSHLMGMFYR | TLRIVDNGIK | PVYVFDGAPP | KLKSGELAKR | FMRKSEAAEA | HEEAKEVGTA |
| 130 | 140 | 150 | 160 | 170 | 180 |
| EEVEKFSRRT | VRVTREHNEE | CKKLLKLMGV | PYIDAPTEAE | AQCAVLARAG | KVYAAASEDM |
| 190 | 200 | 210 | 220 | 230 | 240 |
| DTLCFDSPIL | LRHLTFSEQR | KEPILEIHLD | RVLEGLDMDR | KQFVDLCILL | GCDYLDPIPK |
| 250 | 260 | 270 | 280 | 290 | 300 |
| VGPNTALKLI | RDHGSLEQVV | EAIKSDPKKK | YTIPEDWPYK | EARELFFDPD | VRKADHPDCD |
| 310 | 320 | 330 | 340 | 350 | 360 |
| FKWEAPDVEG | LVKFLVEEKA | FSEDRVRNAA | ARLQKNLKTA | QQSRLEGFFK | PIAKTEQEKA |
| 370 | 380 | 390 | |||
| VLKRKHEEKL | ELQKKKKKED | AKAKKEAKSK | PRGTT |