A0R3R7
Gene name |
ligD (MSMEG_5570, MSMEI_5419) |
Protein name |
Multifunctional non-homologous end joining protein LigD |
Names |
NHEJ DNA polymerase |
Species |
Mycolicibacterium smegmatis (strain ATCC 700084 / mc(2)155) (Mycobacterium smegmatis) |
KEGG Pathway |
msm:MSMEG_5570 |
EC number |
6.5.1.1: Forming phosphoric ester bonds |
Protein Class |
|
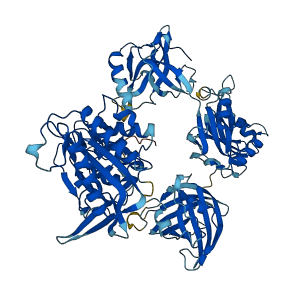
Descriptions
The autoinhibited protein was predicted that may have potential autoinhibitory elements via cis-regPred.
Autoinhibitory domains (AIDs)
Target domain |
|
Relief mechanism |
|
Assay |
cis-regPred |
Accessory elements
No accessory elements
Autoinhibited structure

Activated structure
1 structures for A0R3R7
| Entry ID | Method | Resolution | Chain | Position | Source |
|---|---|---|---|---|---|
| AF-A0R3R7-F1 | Predicted | AlphaFoldDB |
No variants for A0R3R7
| Variant ID(s) | Position | Change | Description | Diseaes Association | Provenance |
|---|---|---|---|---|---|
| No variants for A0R3R7 | |||||
No associated diseases with A0R3R7
5 regional properties for A0R3R7
Functions
| Description | ||
|---|---|---|
| EC Number | 6.5.1.1 | Forming phosphoric ester bonds |
| Subcellular Localization |
|
|
| PANTHER Family | ||
| PANTHER Subfamily | ||
| PANTHER Protein Class | ||
| PANTHER Pathway Category | No pathway information available | |
No GO annotations of cellular component
| Name | Definition |
|---|---|
| No GO annotations for cellular component |
6 GO annotations of molecular function
| Name | Definition |
|---|---|
| ATP binding | Binding to ATP, adenosine 5'-triphosphate, a universally important coenzyme and enzyme regulator. |
| DNA binding | Any molecular function by which a gene product interacts selectively and non-covalently with DNA (deoxyribonucleic acid). |
| DNA ligase (ATP) activity | Catalysis of the reaction: ATP + deoxyribonucleotide(n) + deoxyribonucleotide(m) = AMP + diphosphate + deoxyribonucleotide(n+m). |
| DNA-directed DNA polymerase activity | Catalysis of the reaction: deoxynucleoside triphosphate + DNA(n) = diphosphate + DNA(n+1); the synthesis of DNA from deoxyribonucleotide triphosphates in the presence of a DNA template and a 3'hydroxyl group. |
| exonuclease activity | Catalysis of the hydrolysis of ester linkages within nucleic acids by removing nucleotide residues from the 3' or 5' end. |
| metal ion binding | Binding to a metal ion. |
2 GO annotations of biological process
| Name | Definition |
|---|---|
| DNA recombination | Any process in which a new genotype is formed by reassortment of genes resulting in gene combinations different from those that were present in the parents. In eukaryotes genetic recombination can occur by chromosome assortment, intrachromosomal recombination, or nonreciprocal interchromosomal recombination. Interchromosomal recombination occurs by crossing over. In bacteria it may occur by genetic transformation, conjugation, transduction, or F-duction. |
| double-strand break repair via nonhomologous end joining | The repair of a double-strand break in DNA in which the two broken ends are rejoined with little or no sequence complementarity. Information at the DNA ends may be lost due to the modification of broken DNA ends. This term covers instances of separate pathways, called classical (or canonical) and alternative nonhomologous end joining (C-NHEJ and A-NHEJ). These in turn may further branch into sub-pathways, but evidence is still unclear. |
No homologous proteins in AiPD
| UniProt AC | Gene Name | Protein Name | Species | Evidence Code |
|---|---|---|---|---|
| No homologous proteins | ||||
| 10 | 20 | 30 | 40 | 50 | 60 |
| MARHPWGMER | YERVRLTNPD | KVLYPATGTT | KAEVFDYYLS | IAQVMVPHIA | GRPVTRKRWP |
| 70 | 80 | 90 | 100 | 110 | 120 |
| NGVAEEAFFE | KQLASSAPSW | LERGSITHKS | GTTTYPIINT | REGLAWVAQQ | ASLEVHVPQW |
| 130 | 140 | 150 | 160 | 170 | 180 |
| RFEDGDQGPA | TRIVFDLDPG | EGVTMTQLCE | IAHEVRALMT | DLDLETYPLT | SGSKGLHLYV |
| 190 | 200 | 210 | 220 | 230 | 240 |
| PLAEPISSRG | ASVLARRVAQ | QLEQAMPKLV | TATMTKSLRA | GKVFLDWSQN | NAAKTTIAPY |
| 250 | 260 | 270 | 280 | 290 | 300 |
| SLRGRDHPTV | AAPRTWDEIA | DPELRHLRFD | EVLDRLDEYG | DLLAPLDADA | PIADKLTTYR |
| 310 | 320 | 330 | 340 | 350 | 360 |
| SMRDASKTPE | PVPKEIPKTG | NNDKFVIQEH | HARRLHYDLR | LERDGVLVSF | AVPKNLPETT |
| 370 | 380 | 390 | 400 | 410 | 420 |
| AENRLAVHTE | DHPIEYLAFH | GSIPKGEYGA | GDMVIWDSGS | YETEKFRVPE | ELDNPDDSHG |
| 430 | 440 | 450 | 460 | 470 | 480 |
| EIIVTLHGEK | VDGRYALIQT | KGKNWLAHRM | KDQKNARPED | FAPMLATEGS | VAKYKAKQWA |
| 490 | 500 | 510 | 520 | 530 | 540 |
| FEGKWDGYRV | IIDADHGQLQ | IRSRTGREVT | GEYPQFKALA | ADLAEHHVVL | DGEAVALDES |
| 550 | 560 | 570 | 580 | 590 | 600 |
| GVPSFGQMQN | RARSTRVEFW | AFDILWLDGR | SLLRAKYSDR | RKILEALADG | GGLIVPDQLP |
| 610 | 620 | 630 | 640 | 650 | 660 |
| GDGPEAMEHV | RKKRFEGVVA | KKWDSTYQPG | RRSSSWIKDK | IWNTQEVVIG | GWRQGEGGRS |
| 670 | 680 | 690 | 700 | 710 | 720 |
| SGIGALVLGI | PGPEGLQFVG | RVGTGFTEKE | LSKLKDMLKP | LHTDESPFNA | PLPKVDARGV |
| 730 | 740 | 750 | 760 | ||
| TFVRPELVGE | VRYSERTSDG | RLRQPSWRGL | RPDKTPDEVV | WE |